
Natural Resources
Conservation Service
Ecological site FX052X01X165
Thin Claypan (Tcp)
Dry Grassland
Last updated: 5/08/2025
Accessed: 09/19/2026
-
Search


Major Land Resource Area or ecological site by name and/or ID.
PreviousSectionsNextGeneral information
Provisional. A provisional ecological site description has undergone quality control and quality assurance review. It contains a working state and transition model and enough information to identify the ecological site.
Click to explore map
Figure 1. Mapped extent
Areas shown in blue indicate the maximum mapped extent of this ecological site. Other ecological sites likely occur within the highlighted areas. It is also possible for this ecological site to occur outside of highlighted areas if detailed soil survey has not been completed or recently updated.
MLRA notes
Major Land Resource Area (MLRA): 052X–Brown Glaciated Plains
The Brown Glaciated Plains, MLRA 52, is an expansive, agriculturally and ecologically significant area consisting of around 14.5 million acres that stretches across 350 miles from east to west, encompassing portions of 15 counties in north-central Montana. This region represents the southwestern limit of the Laurentide Ice Sheet and is considered to be the driest and westernmost area within the vast network of glacially-derived prairie pothole landforms of the northern Great Plains. The elevation ranges from 2,000 feet (610 meters) to 4,600 feet (1,400 meters).
Soils are primarily Mollisols but Entisols, Inceptisols, Alfisols and Vertisols are also common. Till from continental glaciation is the predominant parent material, but alluvium and bedrock are also frequently encountered. Till deposits are typically less than 50 feet thick and, in some areas, glacially deformed bedrock can be found at or near the soil surface (Soller, 2001). Underlying sedimentary bedrock largely consisting of Cretaceous shale, sandstone and mudstone (Vuke et al., 2007) is commonly exposed on hillslopes, particularly along drainageways. Significant alluvial deposits occur along glacial outwash channels and major drainages, which include portions of the Missouri, Teton, Marias, Milk and Frenchman Rivers. Large glacial lakes, particularly in the western half of the MLRA, deposited clayey and silty lacustrine sediments (Fullerton et al., 2013).
Much of the western portion of this MLRA was glaciated towards the end of the Wisconsin age with the maximum glacial extent occurring approximately 20,000 years ago (Fullerton et al., 2004). The result is a geologically young landscape that is predominantly a level till plain interspersed with lake plains and dominated by soils in the Mollisol and Vertisol orders. These soils are very productive and generally are well-suited to dryland farming. Much of this area is aridic-ustic and crop-fallow dryland wheat farming is the predominant land use, with rangeland typically being found on steep hillslopes along drainages.
Rangeland, much of it is native mixed grass prairie, increases in abundance in the eastern half of the MLRA. The Wisconsin-age till in the north-central part of this area typically formed large disintegration moraines with steep slopes and numerous poorly drained potholes. A large portion of Wisconsin-age till that is found on this type of terrain, which typically be optimal for farming, has large amounts of less-suitable sodium-affected Natrustalfs. Significant portions of Blaine, Phillips, and Valley Counties were glaciated approximately 150,000 years ago during the Illinoisan age and, due to erosion and dissection of the landscape, much of these areas have steeper slopes and more exposed bedrock than areas glaciated during the Wisconsin age (Fullerton et al., 1986).
While much of the rangeland in the aridic ustic portion of MLRA 52 is classified as belonging to the ‘dry grassland’ climatic zone, sites in portions of southern MLRA 52 may belong to the ‘dry shrubland’ climatic zone. The dry shrubland zone represents the northernmost extent of big sagebrush (Artemisia tridentata) steppe on the Great Plains. As similar soils occur in both the southern and northern portions of the MLRA, it is currently hypothesized that climate is the primary driving factor affecting big sagebrush distribution in this area, but the precise factors have so far proven to be elusive and are, for the time of this writing, not yet fully understood.
Sizable tracts of largely unbroken rangeland in the eastern half of the MLRA and adjacent southern Saskatchewan are home to the Northern Montana Population of Greater Sage Grouse (Centrocercus urophasianus) and large portions of this area are considered to be a Priority Area for Conservation (PAC) by the U.S. Fish and Wildlife Service (U.S. Fish and Wildlife Service, 2013). This population is unique among sage grouse populations in the fact that many individuals overwinter in the big sagebrush steppe (dry shrubland) in the southern portion of the MLRA and then migrate to the northern portion of the MLRA which lacks big sagebrush (dry grassland) to spend rest of the year (Smith, 2013).
Areas of the till plain near the Bearspaw Mountains, Highwood Mountains, Sweetgrass Hills, and Rocky Mountain foothills are at higher elevation, receive higher amounts of precipitation, and have a typic-ustic moisture regime. These areas have significantly more rangeland production than the drier aridic-ustic portions of the MLRA and have enough moisture to produce crops annually as opposed to biennially in the drier areas. Ecological sites in this higher precipitation area are classified as the moist grassland climatic zone.Classification relationships
NRCS Soil Geography Hierarchy
Land Resource Region: Northern Great Plains
Major Land Resource Area: 52
Climatic Zone: Dry Grassland
National Hierarchical Framework of Ecological Units (Cleland et al., 1997; Nesser et al., 1997; McNab et al., 2007)
• Domain: Dry
• Division: Temperate Steppe
• Province: Great Plains-Palouse Dry Steppe Province 331
• Section: Northwestern Glaciated Plains 331D
• Subsection: Montana Glaciated Plains 331Dh
• Landtype association/Landtype phase: N/A
National Vegetation Classification Standard (Federal Geographic Data Committee, 2008)
• Class: Mesomorphic Shrub and Herb Vegetation Class (2)
• Subclass: Temperate and Boreal Grassland and Shrubland Subclass (2.B)
• Formation: Temperate Grassland, Meadow, and Shrubland Formation (2.B.2)
• Division: Great Plains Grassland and Shrubland Division (2.b.2.Nb)
• Macrogroup: Hesperostipa comata – Pascopyrum smithii – Festuca hallii Grassland Macrogroup (2.B.2.Nb.2)
• Group: Pascopyrum smithii – Hesperostipa comata – Schizachyrium scoparium – Bouteloua spp. Mixedgrass Prairie Group (2.B.2.Nb.2.c)
• Alliance: Pascopyrum smithii – Nassella viridula Northwestern Great Plains Herbaceous Alliance
• Association: Pascopyrum smithii –Bouteloua gracilis – Carex filifolia Herbaceous Vegetation
EPA Ecoregions
• Level 1: Great Plains (9)
• Level 2: West-Central Semi-Arid Prairies (9.3)
• Level 3: Northwestern Glaciated Plains (42)
• Level 4: North Central Brown Glaciated Plains (42o) and Glaciated Northern Grasslands (42j)Ecological site concept
The Thin Claypan Dry Grassland ecological site occurs on till plains, moraines and fans, generally on slopes less than eight percent or less. The site is characterized by a dense root-restricting layer (evidenced by columnar structure) that is between one (1) and four (4) inches from the soil surface. The surface texture is typically loam over clay or clay loam. Vegetation is dominated by western wheatgrass (Pascopyrum smithii) and/or thickspike wheatgrass (Elymus lanceolatus). Less common grasses include plains reedgrass (Calamagrostis montanensis), blue grama (Bouteloua gracilis), prairie Junegrass (Koeleria macrantha) and Sandberg bluegrass (Poa secunda). Silver sagebrush is the most common shrub. This site is typically associated with Panspot and Claypan ecological sites. Figure 1 illustrates the distribution of this ecological site based on current data. This map is approximate, is not intended to be definitive, and may be subject to change. Field verification using the appropriate MLRA key is required for proper identification of this ecological site.
Associated sites
FX052X01X006 Claypan (Cp) Dry Grassland
Claypan is found on higher micro topography than Thin Claypan Dry Grassland, but lower than Loamy.
FX052X01X032 Loamy (Lo) Dry Grassland
Loamy is found on the highest micro topography whereas Thin Claypan Dry Grassland is much lower.
FX052X01X145 Panspot (Pn) Dry Grassland
Panspot is found on the lowest micro topography whereas Thin Claypan Dry Grassland occupies higher positions.
Similar sites
FX052X03X165 Thin Claypan (Tcp) Dry Shrubland
Differs from Thin Claypan Dry Grassland in that annual temperatures are slightly warmer and site supports big sagebrush rather than silver sagebrush.
FX052X01X145 Panspot (Pn) Dry Grassland
Differs from Thin Claypan Dry Grassland in that the root restricting layer (evidenced by columnar structure) is 1 inch or less from the surface.
FX052X01X006 Claypan (Cp) Dry Grassland
Differs from Thin Claypan Dry Grassland in that the root restricting layer (evidenced by columnar structure) is greater than 4 inches to 10 inches below the soil surface.
FX052X01X032 Loamy (Lo) Dry Grassland
Differs from Thin Claypan Dry Grassland in that the root restricting layer (evidenced by columnar structure) is either absent or greater than 10 inches below the soil surface.
Table 1. Dominant plant species
Tree Not specified
Shrub Not specified
Herbaceous (1) Pascopyrum smithii
(2) Bouteloua gracilisLegacy ID
R052XY165MT
Physiographic features
The Thin Claypan Dry Grassland ecological site is a common ecological site occurring on moraines, outwash fans and terraces. This site is extensive across MLRA 52 but is most prevalent on the Havre lobe and the contiguous Malta sublobe, which, when combined, stretch from southeastern Alberta and southwestern Saskatchewan through northeastern Hill, central Blaine and southern Phillips Counties. Much of this lobe consists of an extensive ground moraine with slopes of zero to four percent. The till incorporated physical and chemical properties of the underlying clayey Bearpaw shale, which in MLRA 52 tends to have appreciable amounts of sodium, magnesium and calcium sulfates but little to no calcium carbonate.
It is hypothesized that during and immediately after deglaciation, the combination of water-restricting bedrock underlying the sodium-rich clayey till at depths of 10 feet or less combined with the gentler slopes of the till plain created an ideal situation where water could pond and move, by matric potential to concentrate enough salts to create the natric horizon and its distinctive columnar structure (Miller and Brierly, 2011). The present-day hydrology of this site lacks a water table. As is the case with the Thin Claypan site, complex micro relief is normal on landforms dominated by natric soils. Figure 4 shows a landscape cross section of the natric catena and the position of the Thin Claypan in relation to other sites.
Figure 2. Extent of the Thin Claypan Dry Grassland Ecological Site within MLRA 52 based on soil mapunit component.

Figure 3. Landscape cross-section of the Natric Catena
Table 2. Representative physiographic features
Landforms (1) Till plain > Moraine
(2) Till plain > Outwash fan
(3) Terrace
Elevation 2000 – 3870 ft Slope 0 – 8 % Aspect Aspect is not a significant factor Table 3. Representative physiographic features (actual ranges)
Elevation 2000 – 3870 ft Slope 0 – 14 % Climatic features
The Brown Glaciated Plains is a semi-arid region with a temperate continental climate that is characterized by frigid winters and warm to hot summers (Cooper et al., 2001). The average frost-free period for this ecological site is 120 days. The majority of precipitation occurs as steady, soaking, frontal system rains in late spring to early summer. Summer rainfall comes mainly from convection thunderstorms that typically deliver scattered amounts of rain in intense bursts. These storms may be accompanied by damaging winds and large-diameter hail and result in flash flooding along low-order streams. Severe drought occurs on average in two (2) out of every 10 years. Annual precipitation ranges from 10 to 14 inches, and 70 to 80 percent of this occurs during the growing season (Cooper et al., 2001). Extreme climatic variations, especially droughts, have the greatest influence on species cover and production (Coupland, 1958, 1961; Biondini et al., 1998).
During the winter months, the western half of MLRA 52 commonly experiences Chinook winds, which are strong west to southwest surface winds accompanied by abrupt increases in temperature. The chinook winds are strongest on the western boundary of the MLRA near the Rocky Mountain foothills and decrease eastward. In addition to producing damaging winds, prolonged chinook episodes can result in drought or vegetation kills due to the reaction of plants to a “false spring” (Oard, 1993).Table 4 Representative climatic features
Frost-free period (characteristic range) 110-130 days Freeze-free period (characteristic range) 130-150 days Precipitation total (characteristic range) 10-10 in Frost-free period (average) 120 days Freeze-free period (average) 140 days Precipitation total (average) 10 in BarLineFigure 4. Monthly precipitation range
BarLineFigure 5. Monthly minimum temperature range
BarLineFigure 6. Monthly maximum temperature range
BarLineFigure 7. Monthly average minimum and maximum temperature
Figure 8. Annual precipitation pattern
Figure 9 Annual average temperature pattern
Climate stations used
-
(1) CARTER 14 W [USC00241525], Floweree, MT
-
(2) CHESTER [USC00241692], Chester, MT
-
(3) TIBER DAM [USC00248233], Chester, MT
-
(4) HARLEM [USC00243929], Harlem, MT
-
(5) MALTA 7 E [USC00245338], Malta, MT
-
(6) TURNER 11N [USC00248415], Turner, MT
-
(7) CONRAD [USC00241974], Conrad, MT
-
(8) SHELBY [USC00247500], Shelby, MT
-
(9) GLASGOW [USW00094008], Glasgow, MT
-
(10) HAVRE CITY CO AP [USW00094012], Havre, MT
">Influencing water features
This site is not influenced by a groundwater table. Infiltration is limited by a dense clay layer near the soil surface. Moisture loss through potential evapotranspiration exceeds precipitation for the majority of the growing season. Except for May and June, the site is generally in a state of moisture deficit.
Soil features
The soil that best represents the central concept for this ecological site is the benchmark Elloam series, which covers over 780,000 acres of MLRA 52. This soil is in the Natrustalfs Great Group and is characterized by a surface horizon that lacks enough organic matter to have a mollic epipedon and by a dense, root-limiting, non-cemented restrictive layer one to four inches below the soil surface. This restrictive layer is referred to as a natric horizon and is essentially an argillic horizon that has been affected by sodium salts. The natric horizon exhibits a distinctive columnar structure that is especially visible when the soil is dry. Elloam is a fine family and has smectitic mineralogy. Clayey till (28 to 42 percent clay) is the typical parent material for this series, but the Thin Claypan ecological sit may also occur on soils derived from glaciofluvial deposits, shale residuum, or till over residuum. The soil moisture regime for this and all soils in this ecological site concept is ustic bordering on aridic, which means that the soils are moist in some or all parts for either 180 cumulative days or 90 consecutive days during the growing season but are dry in some or all parts for over 90 cumulative days. These soils have a frigid soil temperature regime (Soil Survey Staff, 2014).
Surface textures found in this site are most frequently loam but can range from fine sandy loam to silty clay loam and usually contain between 15 and 30 percent clay. The underlying natric horizons typically contain 35 to 50 percent clay and have clay, clay loam or silty clay loam textures. Organic matter in the surface horizon typically ranges from one to two percent and moist colors vary from brown (10YR 5/3) to dark grayish brown (10YR 4/2). The surface of these soils does not typically react with hydrochloric acid. The depth to secondary carbonates and soluble sulfate salts is usually between five and eight inches below the soil surface. Calcium carbonate equivalent in the soil surface five inches is typically less than five percent and typically less than 10 percent in lower horizons. In the soil surface 20 inches, electrical conductivity is, at some point, more than two and less than eight and the sodium absorption ratio is typically less than 15. These salts lower the amount of plant-available water. Soil pH classes are moderately acidic to slightly alkaline in the surface horizon and neutral to strongly alkaline in the subsurface horizons. The soil depth class for this site can be moderately deep (between 20 and 40 inches to bedrock) in places where bedrock is present but is typically very deep (greater than 60 inches to bedrock). Coarse fragments are less than 35 percent in the upper 20 inches of soil and are typically less than 15 percent.
Figure 10. Typical Soil Profile
Table 5. Representative soil features
Parent material (1) Till
(2) Glaciofluvial deposits
(3) Residuum
Surface texture (1) Loam
(2) Fine sandy loam
(3) Silty clay loam
Family particle size (1) Fine
Drainage class Well drained Depth to restrictive layer 1 – 4 in Soil depth 60 – 72 in Available water capacity
(0-40in)3 – 4.7 in Calcium carbonate equivalent
(0-5in)0 – 4 % Electrical conductivity
(0-20in)2 – 8 mmhos/cm Sodium adsorption ratio
(0-20in)2 – 15 Soil reaction (1:1 water)
(0-40in)6.1 – 8.4 Subsurface fragment volume <=3"
(0-20in)0 – 14 % Subsurface fragment volume >3"
(0-20in)0 – 14 % Table 6. Representative soil features (actual values)
Drainage class Well drained Depth to restrictive layer 1 – 4 in Soil depth 20 – 72 in Available water capacity
(0-40in)3 – 4.7 in Calcium carbonate equivalent
(0-5in)0 – 14 % Electrical conductivity
(0-20in)0 – 8 mmhos/cm Sodium adsorption ratio
(0-20in)2 – 15 Soil reaction (1:1 water)
(0-40in)5.6 – 9 Subsurface fragment volume <=3"
(0-20in)0 – 34 % Subsurface fragment volume >3"
(0-20in)0 – 34 % Ecological dynamics
The information in this ecological site description, including the state-and-transition model (STM), was developed based on historical data, current field data, professional experience, and a review of the scientific literature. As a result, all possible scenarios or plant species may not be included. Key indicator plant species, disturbances, and ecological processes are described to inform land management decisions.
The Thin Claypan Dry Grassland ecological site in MLRA 52 Dry Grassland consists of five states: The Reference state (1.0), the Shortgrass state (2.0), the Invaded state (3.0), the Annual Cropland state (4.0), and the Post Cropland state (5.0).
The presumed Historic Reference Community of the Thin Claypan Dry Grassland ecological site was dominated by mid-statured, cool-season perennial rhizomatous wheatgrasses. Short-statured, cool-season grasses, particularly prairie Junegrass and Sandberg bluegrass were common on these sites although cover and production were low. The mat-forming, warm-season perennial grass, blue grama was also an important component of this site, although its contribution varied with climate and disturbance. Due to the impermeable nature of the soil, deeper-rooted bunchgrasses such as needle and thread (Hesperostipa comata) are not well-adapted to this site (Coupland, 1961; Coupland and Johnson, 1965), although needle and thread did occur as a minor component of the plant community on portions of the site with thicker soil horizons. The species composition and cover of forbs were low on this site. The subshrub prairie, or fringed, sagewort (Artemsia frigida) also had low cover on this site. Plains pricklypear (Opuntia polyacantha) was uncommon on this site. Lesser spikemoss (Selaginella densa), more locally known and hereinafter referred to as dense clubmoss also occurs on this site, but its cover was highly variable and dependent upon fire frequency, climate, and grazing.
Plant communities associated with the Thin Claypan Dry Grassland ecological site evolved under the combined influences of climate, grazing, and fire. Extreme climatic variability results in frequent droughts, which can have the greatest influence on the relative contribution of species cover and production (Coupland, 1958, 1961; Biondini et al., 1998; Umbanhowar, 2004). Due to the dominance of cool-season grasses, annual production is highly dependent upon mid- to late-spring precipitation (Heitschmidt and Vermeire, 2005; Anderson, 2006).
Native grazers also shaped these plant communities. Bison (Bison bison) were the dominant historic grazers, but pronghorn (Antilocarpa americana), elk (Cervus canadensis), and deer (Odocoileus spp.) were also common. Additionally, small mammals such as prairie dogs (Cynomys spp.), and ground squirrels (Urocitellus spp.) also influenced this plant community (Salo et al., 2004). Grasshoppers and periodic outbreaks of Rocky Mountain locusts (Melanoplus spretus) also played an important role in the ecology of these communities (Lockwood, 2004).
The historic reference community experienced relatively frequent lightning-caused fires with estimated fire return intervals of six to 25 years (Bragg, 1995). Historically, Native Americans also set frequent fires. The majority of lightning-caused fires occurred in July and August, whereas Native Americans typically set fires during spring and fall to correspond with the movement of bison (Higgins, 1986).
Frequent fire is no longer a major disturbance to this ecological site due to fire suppression and cessation of fires ignited by Native Americans. This lack of frequent fires has resulted in an increase in litter accumulation in some areas, providing ideal conditions for seed germination and seedling establishment of non-native annual brome species, such as field, or Japanese, brome (Bromus arvensis; Whisenant, 1990). These species have become naturalized in relatively undisturbed grasslands, and their presence can reduce the production of cool-season perennial grasses (Ogle et al., 2003; Harmoney, 2007; Haferkamp et al., 1997). Fire suppression may also be one mechanism that triggers increased cover of dense clubmoss (Rowe, 1969; Shay et al., 2001). The cover of dense clubmoss is generally less on recently burned sites; however, its abundance may also vary greatly from site to site without discernable reason (Dix, 1960; Wilson and Shay, 1990). In general, mechanisms affecting dense clubmoss abundance are not well understood and require further investigation.
Improper grazing of this site can result in a reduction in the cover of the cool-season wheatgrasses and, eventually a decrease in other cool-season grasses and an increase in blue grama (Smoliak et al., 1972; Smoliak, 1974). Periods of extended drought can reduce mid-statured, cool-season, rhizomatous wheatgrasses, shifting the species composition of this community to one dominated by blue grama (Coupland, 1958, 1961).
Further degradation of the site due to improper grazing can result in a community dominated by shortgrasses such as blue grama and Sandberg bluegrass (Adams et al., 2013). Cover of mid-statured rhizomatous grasses and bunchgrasses is severely reduced or absent. Cover of prairie sagewort can increase.
The Thin Claypan Dry Grassland ecological site is not generally considered suitable for cropland. However, a good portion of it has been converted to annual cropland despite the soil limitations. Seeding of introduced grasses, particularly crested wheatgrass (Agropyron cristatum), was a common practice on eroded and abandoned agricultural areas after the droughts of the 1930s (Rogler and Lorenz, 1983). Crested wheatgrass is a highly drought-tolerant and competitive cool-season, perennial bunchgrass (DeLuca and Lesica, 1986). Crested wheatgrass can invade relatively undisturbed grasslands, reducing cover and production of native cool-season midgrasses (Heidinga and Wilson, 2002; Henderson and Naeth, 2005). Russian wildrye (Psathyrostachys juncea), though less widespread, was introduced in the 1950s to provide forage for livestock (Dormaar et al., 1995). Although Russian wildrye is typically planted in monocultures, this species is not considered invasive. Under ideal conditions, it may be able to spread into adjacent degraded plant communities (Ogle et al., 2012), but such conditions are unlikely in MLRA 52.
When this site is taken out of production, the site is either allowed to revert to perennial grassland or is seeded with introduced species. Sites left to undergo natural plant succession after cultivation can, over several decades, support blue grama and cool-season shortgrasses, although the cover and production of these species are lower than in the Reference state. However, those sites seeded with non-native species, particularly crested wheatgrass, may persist as this cover type indefinitely (Christian and Wilson, 1999).
The STM diagram suggests possible pathways that plant communities on this site may follow as a result of a given set of ecological processes and management. The site may also support states not displayed in the STM diagram. Landowners and land managers should seek guidance from local professionals before prescribing a particular management or treatment scenario.
Plant community responses vary across this MLRA due to variability in weather, soil, and aspect. The Reference community may not necessarily be the management goal. The lists of plant species, species cover, and production values are representative. These are not intended to cover the full range of conditions, species, and responses for the site. Cover values are presented as foliar cover unless otherwise noted. Species composition by dry weight is provided when describing the herbaceous plant communities.State and transition model
More interactive model formats are also available. View Interactive Models
Click on state and transition labels to scroll to the respective textT1A - prolonged drought, improper grazing, or a combination of these factors T1B - The introduction of aggressive perennial grasses (mostly crested wheatgrass) T1C - Conversion to annual cropland R2A - range seeding, grazing land mechanical treatment, timely moisture, proper grazing management (management intensive and costly) T2A - introduction of weedy species; combined with drought and/or improper grazing management T2B - conversion to annual cropland T3A - conversion to annual cropland T4A - cessation of annual cropping T5A - conversion to annual cropland State 1 submodel, plant communities
1.1A - drought, improper grazing management, multiple fires in close succession 1.2A - timely moisture, proper grazing management State 2 submodel, plant communities
State 3 submodel, plant communities
State 4 submodel, plant communities
State 5 submodel, plant communities
State 1
ReferenceThe Reference state consists of two communities. The dynamics of this state are driven by the combined influences of climate, grazing, and fire. Dense clubmoss may be present in any of the communities within this state; however, its density is highly variable and the dynamics of this species are not well understood (Romo and Bai, 2004; Romo, 2011). Research has shown that its density is affected by drought, fire, and hoof action by grazing animals (Coupland, 1950; VanDyne and Vogel, 1967; Clarke et al., 1947). However, its abundance may vary greatly from site to site without discernable reason. In general, this state is characterized by a predominance of mid-statured, cool-season rhizomatous grasses. As ecological conditions decline; mid-statured grasses decrease and are replaced by short-statured grasses such as blue grama and Sandberg bluegrass. Plant Community 1.2 is dominated by blue grama and rhizomatous wheatgrasses, although wheatgrasses decrease in this community. Sandberg bluegrass also increases in Plant Community 1.2, as does prairie sagewort. Drought, improper grazing management, or a combination of these factors can transition this state to the Shortgrass state.
Dominant plant species
-
western wheatgrass (Pascopyrum smithii), grass
-
blue grama (Bouteloua gracilis), grass
Community 1.1
Rhizomatous Wheatgrass
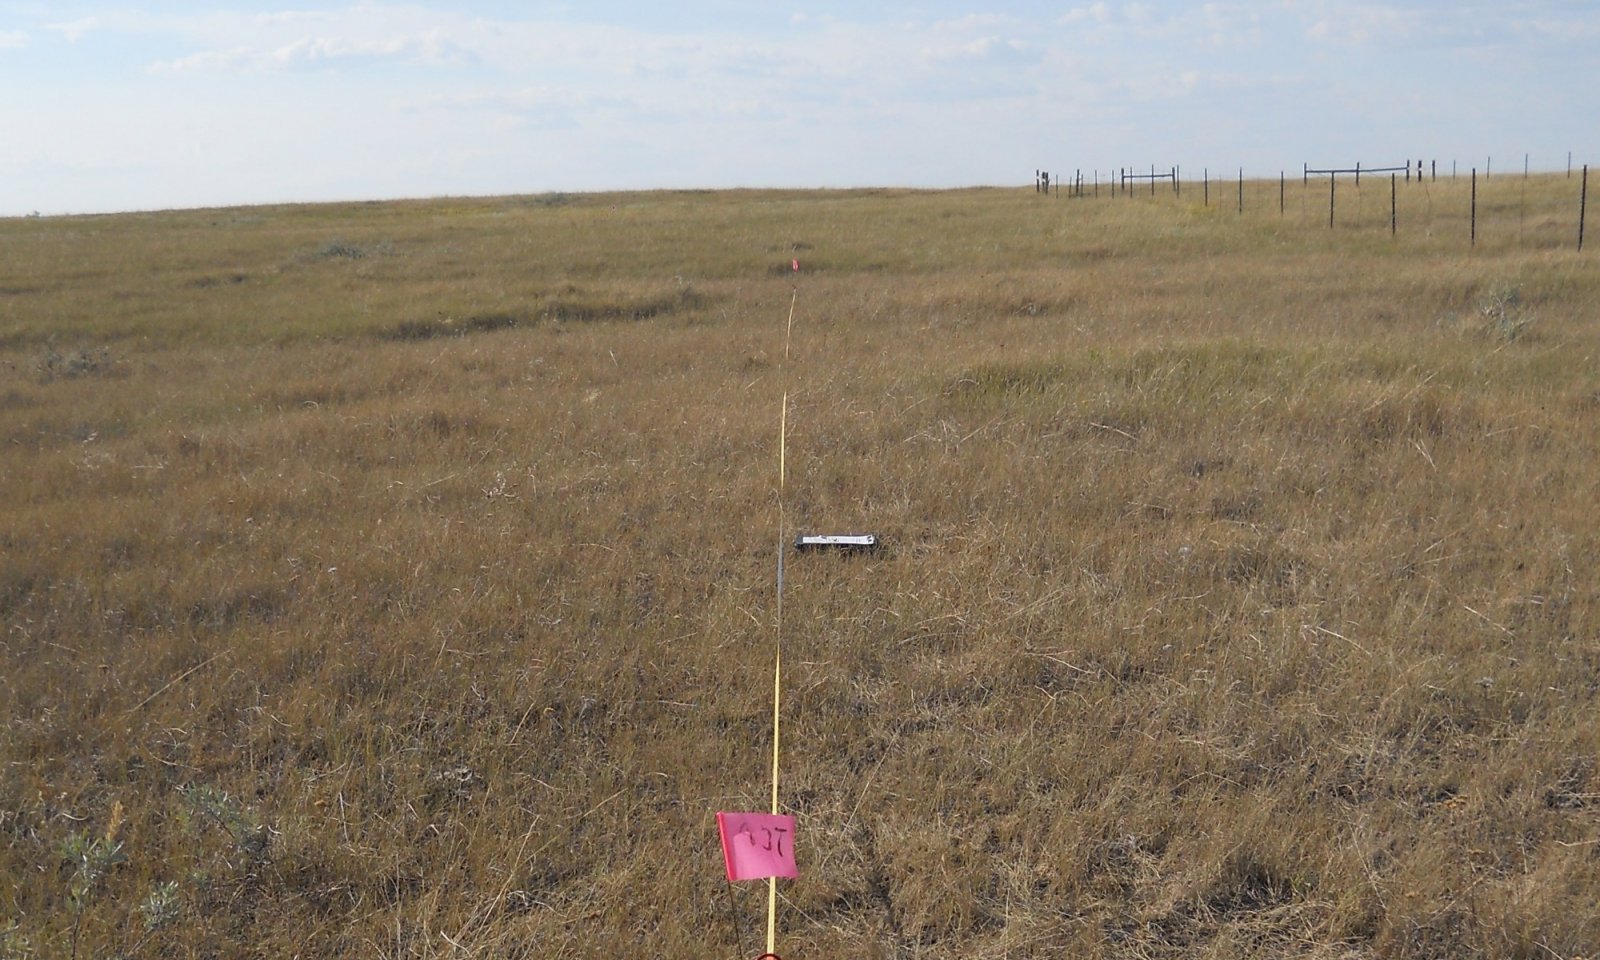
Figure 11. Figure 7 Rhizomatous Wheatgrass plant community (1.1) for Thin Claypan Dry Grassland ecological site. Elloam Soils. Photo by Montana Natural Heritage Program, Valley County, Montana, August 2012
This plant community is dominated by rhizomatous wheatgrasses. Both western wheatgrass and thickspike wheatgrass can occur in this community, although western wheatgrass is more common due to its greater tolerance to droughty conditions associated with this site (Coupland, 1950).
Short-statured, cool-season grasses, particularly prairie Junegrass and Sandberg bluegrass, are common on these sites although cover and production are low. The mat-forming, warm-season perennial grass, blue grama is also an important component of this site, although its contribution varies with climate and disturbance. Due to the impermeable nature of the soil, deeper-rooted bunchgrasses such as needle and thread are not well-adapted to this site (Coupland, 1961), although needle and thread can occur as a minor component of the plant community on portions of the site with thicker soil horizons. Both the species composition and cover of forbs are typically low on this site, generally five percent cover or less. Common forb species include spiny, or Hood’s, phlox (Phlox hoodii) and scarlet globemallow (Sphaeralcea coccinea). Dense clubmoss cover varies substantially, with some sites having 70 to 80 percent cover and other sites having little or no cover. The subshrub prairie sagewort is common but with low cover. Plains pricklypear is uncommon. The principal shrub on this site, if present, is silver sagebrush, although canopy cover is generally less than five percent.
Non-native annual bromes, particularly field brome, have become naturalized on this ecological site. Cover of annual bromes is typically low, but it can vary significantly from season to season depending on seed germination conditions. Frequent fires can reduce litter accumulation enough to limit field brome germination (Whisenant, 1990). However, long-term fire suppression may result in increased litter accumulation and greater germination of non-native annual bromes.
The following tables characterize the Rhizomatous Wheatgrasses plant community (1.1) by the following elements:
Plant Community Phase Composition and Foliar Cover
Total Annual Production
Ground Surface Cover
Structure
Information in these tables was developed using current field data in conjunction with a review of the scientific literature and professional experience.Dominant plant species
-
western wheatgrass (Pascopyrum smithii), grass
-
blue grama (Bouteloua gracilis), grass
Figure 12. Annual production by plant type (representative values) or group (midpoint values)
Table 7. Annual production by plant type
Plant type Low
(lb/acre)Representative value
(lb/acre)High
(lb/acre)Grass/Grasslike 220 395 625 Forb 40 70 115 Shrub/Vine 10 15 20 Total 270 480 760 Table 8. Ground cover
Tree foliar cover 0% Shrub/vine/liana foliar cover 0-10% Grass/grasslike foliar cover 50-70% Forb foliar cover 0-30% Non-vascular plants 0-0% Biological crusts 0% Litter 20-50% Surface fragments >0.25" and <=3" 0% Surface fragments >3" 0% Bedrock 0% Water 0% Bare ground 0% Table 9. Soil surface cover
Tree basal cover 0% Shrub/vine/liana basal cover 0-0% Grass/grasslike basal cover 0-10% Forb basal cover 0-80% Non-vascular plants 0-10% Biological crusts 0% Litter 0% Surface fragments >0.25" and <=3" 0-10% Surface fragments >3" 0-0% Bedrock 0% Water 0% Bare ground 0-10% Table 10. Canopy structure (% cover)
Height Above Ground (ft) Tree Shrub/Vine Grass/
GrasslikeForb <0.5 – – 5-25% 1-10% >0.5 <= 1 – 0-1% 25-55% – >1 <= 2 – 0-5% 5-10% – >2 <= 4.5 – – – – >4.5 <= 13 – – – – >13 <= 40 – – – – >40 <= 80 – – – – >80 <= 120 – – – – >120 – – – – Figure 13. Plant community growth curve (percent production by month). MT005 , MLRA 52 (cool season dominant). Typically occurs in Reference or Contemporary Reference State.
Jan Feb Mar Apr May Jun Jul Aug Sep Oct Nov Dec J F M A M J J A S O N D 10 25 45 15 5 Community 1.2
Blue Grama and Rhizomatous Wheatgrass
Figure 14. Figure 3. Blue Grama and Rhizomatous Wheatgrass Plant (1.2) Community for Thin Claypan Dry Grassland ecological site. Elloam Soils. Photo by Charles French (Soil Scientist, NRCS), Phillips County, Montana, June 2015
Drought, improper grazing management, multiple fires in close succession, or a combination of these factors can shift the Rhizomatous Wheatgrass community (1.1) towards the Blue Grama and Rhizomatous Wheatgrass community (1.2). This community is characterized by an increase in the warm-season, mat-forming blue grama. The cover of blue grama equals or exceeds wheatgrasses, which decreases in this community. The cool-season, perennial bunchgrass needle and thread becomes rare or is absent. The shortgrass, Sandberg bluegrass and the subshrub, prairie sagewort, increase in this phase. This plant community is considerably less productive than the Rhizomatous Wheatgrass community due to the significant decrease in cool-season rhizomatous wheatgrasses. This plant community can return to the Rhizomatous Wheatgrass community with proper grazing management and normal or above-normal spring precipitation. Continued improper grazing management will drive this community to the Shortgrass state (2).
Pathway 1.1A
Community 1.1 to 1.2
Rhizomatous Wheatgrass
Blue Grama and Rhizomatous WheatgrassDrought, improper grazing management, multiple fires in close succession, or a combination of these factors can shift the Rhizomatous Wheatgrass community (1.1) to the Blue Grama and Rhizomatous Wheatgrass community (1.2). These factors favor an increase in blue grama and a decrease in cool-season midgrasses (Coupland, 1961; Shay et al., 2001; Smith and McDermid, 2014).
Context dependence.Timing of precipitation may affect species composition of perennial grasses.
Pathway 1.2A
Community 1.2 to 1.1
Blue Grama and Rhizomatous Wheatgrass
Rhizomatous WheatgrassThe Blue Grama and Rhizomatous Wheatgrass plant community (1.2) can return to the Rhizomatous Wheatgrass Plant community (1.1) with normal or above-normal spring precipitation and proper grazing management.
Context dependence.Timing of precipitation may affect species composition of perennial grasses.
State 2
ShortgrassThe Shortgrass state consists of two communities. The dynamics of this state are driven by long-term drought, improper grazing management, or a combination of these factors. Rhizomatous wheatgrasses have low production and poor vigor in this state. Prairie sagewort is common. Blue grama increases with long-term improper grazing at the expense of cool-season midgrasses (Coupland, 1961; Biondini and Manske, 1996; Derner and Whitman, 2009). Reductions in stocking rates can reduce blue grama cover and increase the cover of cool-season midgrasses, although this recovery may take decades (Dormaar and Willms, 1990; Dormaar et al., 1994). Dense clubmoss may or may not be present in this state and the dynamics of this species are not well understood. In some cases, it is abundant on heavily grazed areas, but in others, it is rare or absent. Its abundance varies greatly from site to site without a discernable reason, therefore, it is not considered a reliable indicator of past grazing use (Montana State College, 1949). Annual bromes are also present in this state. They are naturalized but usually do not have a significant ecological impact; however, their abundance varies depending on precipitation and germination conditions.
Community 2.1
Blue Grama and Sandberg BluegrassOn sites where clubmoss is not present, the Blue Grama and Sandberg Bluegrass plant community occurs as the result of long-term improper grazing management. This plant community is dominated by the warm-season, mat-forming blue grama and cool-season shortgrasses, particularly Sandberg bluegrass. Long-term improper grazing management has considerably reduced the cover and annual production of this site, changing the structure of this plant community from a mid-statured grassland to a shortgrass community (Derner and Hart, 2007). Cool-season, rhizomatous wheatgrasses have decreased significantly in this phase, and grazing-tolerant species like blue grama, Sandberg bluegrass, and prairie Junegrass have increased. Prairie sagewort also increases in this phase.
Figure 15. Plant community growth curve (percent production by month). MT041 , MLRA 52 (warm season dominant). Typically occurs in the Short Grass State.
Jan Feb Mar Apr May Jun Jul Aug Sep Oct Nov Dec J F M A M J J A S O N D 5 20 50 20 5 Community 2.2
Blue Grama and Dense ClubmossOn sites where clubmoss is present, the Blue Grama and Dense Clubmoss community occurs as the result of long-term improper grazing management. The cool-season rhizomatous wheatgrasses are rare and have low reproductive vigor. The warm-season, mat-forming blue grama and dense clubmoss comprise the dominant basal cover for this phase. Prairie sagewort, Sandberg bluegrass, and prairie Junegrass are also common. Continued improper grazing management combined with the introduction of invasive pasture grasses can drive this community phase to the Invaded state (3).
State 3
InvadedThe Invaded state (3) occurs when invasive plant species, primarily crested wheatgrass, invade adjacent native grassland communities. An estimated 20 million acres of crested wheatgrass have been planted in the western U.S. (Holechek, 1981). Since the 1930s, crested wheatgrass has been planted to improve forage for livestock (Roglers and Lorenz, 1983; Laycock, 1988). Beginning in the mid-1980s, crested wheatgrass was often seeded on lands enrolled in the Conservation Reserve Program (CRP; Roath, 1988; DeLuca and Lesica, 1996). Crested wheatgrass is extremely drought tolerant, establishes readily on a variety of soil types, has high seedling vigor, and provides highly productive early-season forage for livestock (Roglers and Lorenz, 1983). Once established, monocultures of crested wheatgrass can persist for at least 60 years (Krzic et al., 2000; Henderson and Naeth, 2005), as crested wheatgrass stands resist the recruitment of native plant species (Looman and Heinrichs, 1973; Henderson and Naeth, 2005; Fansler and Mangold, 2011).
Crested wheatgrass produces abundant seeds that can dominate the seedbank of invaded grasslands, although crested wheatgrass cover decreases with increasing distance from seeded areas (Henderson and Naeth, 2005; Heidinga and Wilson, 2002). The early growth of crested wheatgrass allows this species to take advantage of early-season soil moisture, which may result in competitive exclusion of native cool-season rhizomatous wheatgrasses and bunchgrasses such as needle and thread and prairie Junegrass (Christian and Wilson, 1999; Heidinga and Wilson, 2002; Henderson and Naeth, 2005). If already established, the warm-season, mat-forming blue grama may compete successfully with crested wheatgrass, although the ability of blue grama to persist in invaded stands is unknown due to its low seed production and narrow germination requirements (Coupland, 1950; Heidinga and Wilson, 2002; Lauenroth et al., 1994). Reduced soil quality, reduced plant species diversity, and simplified structural complexity (Dormaar et al., 1995; Henderson and Naeth, 2005) result in a state that is substantially departed from the Reference state (1).Dominant plant species
-
crested wheatgrass (Agropyron cristatum), grass
-
blue grama (Bouteloua gracilis), grass
Community 3.1
Blue Grama and Crested WheatgrassEncroachment by crested wheatgrass and other invasives common. Rangeland health attributes departed substantially from reference state
Dominant plant species
-
crested wheatgrass (Agropyron cristatum), grass
-
blue grama (Bouteloua gracilis), grass
State 4
Annual CroplandThe Annual Cropland state (4) occurs when land is put into cultivation. Major crops in MLRA 52 include winter and spring wheat, as well as barley.
Community 4.1
CroplandAnnual, cool-season cereal grains such as spring wheat, winter wheat, and barley are common crops which replace native plant communities.
State 5
Post CroplandThe Post Cropland state (5) occurs when cultivated cropland is abandoned and allowed to either re-vegetate naturally or is seeded back to perennial species for livestock grazing or wildlife use. This state can transition back to the Cropland state (4) if the site is returned to cultivation.
Community 5.1
Abandoned CroplandIn the absence of active management, the site can re-vegetate naturally and potentially return to a perennial grassland community over time. Shortly after cropland is abandoned, annual and biennial forbs and annual brome grasses invade the site. The site is highly susceptible to erosion due to the absence of perennial species. Eventually, these pioneering annual species are replaced by perennial forbs and perennial shortgrasses. Depending on the historical management of the site, mid-statured perennial grasses may also return; however, species composition will depend upon the seed bank. Invasion of the site by exotic species, such as crested wheatgrass and annual bromes, will depend upon the site’s proximity to a seed source. Fifty or more years after cultivation, these sites may have species composition similar to phases in the Reference state (1). However, soil quality is consistently lower than conditions before cultivation and a shift to the Reference state (1) is unlikely within a reasonable timeframe (Dormaar and Smoliak, 1985).
Community 5.2
Perennial GrassWhen the site is seeded to perennial forage species, this community phase can persist for several decades. Introduced perennial grasses, in particular, may form monocultures that persist for 60 years or more (Samuel and Hart, 1994). A mixture of native species may also be seeded to provide species composition and structural complexity similar to that of the Reference state (1). However, soil quality conditions have been substantially altered and will not return to pre-cultivation conditions within a reasonable timeframe.
Transition T1A
State 1 to 2The Reference state (1) transitions to the Shortgrass state (2) when cool-season rhizomatous wheatgrasses become rare and contribute little to production. Shortgrasses, particularly the warm-season, mat-forming blue grama, as well as Sandberg bluegrass, dominate the plant community. Prolonged drought, improper grazing practices or a combination of these factors weaken the resilience of the Reference state (1) and drive its transition to the Shortgrass state (2).
Context dependence.Drought may accelerate or exacerbate change. Soils are particularly susceptible to erosion when dry.
Transition T1B
State 1 to 3The Reference state (1) transitions to the Invaded state (3) when aggressive perennial grasses, particularly crested wheatgrass, invade the Reference state (1). These communities are often adjacent to seeded pastures. Exotic plant species dominate the site in terms of cover and production. Site resilience has been substantially reduced and other rangeland health attributes such as the reproductive capacity of native grasses and soil quality have been substantially altered from the Reference state (Henderson and Naeth, 2005; Smoliak and Dormaar, 1985; Dormaar et al., 1995).
Context dependence.Close proximity to a seed source increases the likelihood of encroachment by invasive species.
Transition T1C
State 1 to 4The Reference state (1) will transition to the Cropland state (4) when the site is placed into cultivation with crops such as winter and spring wheat and barley.
Context dependence.Drought may accelerate or exacerbate change. Cropped soils are particularly susceptible to erosion during drought.
Restoration pathway R2A
State 2 to 1Blue grama can resist displacement by other species (Dormaar and Willms, 1990; Laycock, 1991; Dormaar et al., 1994; Lacey et al., 1995). A reduction in livestock grazing pressure alone may not be sufficient to reduce the cover of blue grama in the Shortgrass state (2) (Dormaar and Willms, 1990), and mechanical treatments may be necessary (Hart et al., 1985). Therefore, returning the Shortgrass state (2) to the Reference state (1) can require considerable cost, energy, and time.
Context dependence.Drought may inhibit recovery despite management inputs. Reseedings are more likely to fail during drought.
Transition T2A
State 2 to 3The Shortgrass state (2) transitions to the Invaded state (3) when aggressive perennial grasses such as crested wheatgrass invade the Shortgrass state (2). This transition can occur when native plant communities are adjacent to seeded pastures. Exotic plant species, particularly crested wheatgrass, dominate the site in terms of cover and production. Crested wheatgrass can outcompete native grasses (Vaness and Wilson, 2007), weakening site resilience and impacting rangeland health attributes such as the reproductive capacity of native grasses (Henderson and Naeth, 2005) and soil quality (Smoliak and Dormaar, 1985; Dormaar et al., 1995).
Context dependence.Close proximity to a seed source increases likelihood of encroachment by invasive species.
Transition T2B
State 2 to 4The Shortgrass state (2) transitions to the Cropland state (4) when the site is placed into cultivation with crops such as winter and spring wheat and barley.
Context dependence.Drought may accelerate or exacerbate change. Cropped soils are particularly susceptible to erosion during drought.
Transition T3A
State 3 to 4The transition from the Invaded state (3) to the Annual Cropland state (4) occurs when the site is placed into cultivation with crops such as winter and spring wheat and barley.
Context dependence.Drought may accelerate or exacerbate change. Cropped soils are particularly susceptible to erosion during drought.
Transition T4A
State 4 to 5The transition from the Annual Cropland state (4) to the Post Cropland state (5) occurs with the cessation of cultivation. The site may also be seeded to perennial forage species such as crested wheatgrass and alfalfa or a mix of native species.
Context dependence.Drought may inhibit recovery despite management inputs. Reseedings are more likely to fail during drought.
Transition T5A
State 5 to 4Tillage or application of herbicide followed by seeding of cultivated crops, such as winter wheat, spring wheat, and barley, transitions the Post Cropland state (5) to the Cropland state (4).
Context dependence.Drought may accelerate or exacerbate change. Cropped soils are particularly susceptible to erosion during drought.
Additional community tables
Table 11. Community 1.1 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Grass/Grasslike1 Mid stature, cool season rhizomatous grasses 155–430 western wheatgrass PASM Pascopyrum smithii 125–340 21–65 thickspike wheatgrass ELLA3 Elymus lanceolatus 125–340 21–65 plains reedgrass CAMO Calamagrostis montanensis 30–90 4–8 2 Mid stature, cool season bunchgrasses 0–40 needle and thread HECO26 Hesperostipa comata 0–40 0–5 3 Short stature graminoids 50–115 blue grama BOGR2 Bouteloua gracilis 20–50 2–10 prairie Junegrass KOMA Koeleria macrantha 15–45 1–5 sedge CAREX Carex 15–40 1–5 Sandberg bluegrass POSE Poa secunda 0–10 0–5 4 Other Native Graminoids 15–40 Grass, perennial 2GP Grass, perennial 15–40 1–5 Forb5 Perennial forbs 40–115 Forb, native 2FN Forb, native 20–40 1–5 common yarrow ACMI2 Achillea millefolium 15–30 1–10 scarlet globemallow SPCO Sphaeralcea coccinea 5–15 0–2 American vetch VIAM Vicia americana 0–15 0–2 pussytoes ANTEN Antennaria 5–10 0–2 spiny phlox PHHO Phlox hoodii 0–5 0–1 rough false pennyroyal HEHI Hedeoma hispida 0–5 0–1 Shrub/Vine6 Native Shrubs and Halfshrubs 8–15 silver sagebrush ARCA13 Artemisia cana 0–15 0–5 prairie sagewort ARFR4 Artemisia frigida 8–15 0–1 broom snakeweed GUSA2 Gutierrezia sarothrae 0–5 0–1 7 Cactus 2–5 plains pricklypear OPPO Opuntia polyacantha 2–5 1–2 Table 12. Community 1.2 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 13. Community 2.1 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 14. Community 2.2 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 15. Community 3.1 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 16. Community 4.1 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 17. Community 5.1 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 18. Community 5.2 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Interpretations
Animal community
Grassland communities within the Thin Claypan Dry Grassland ecological site of MLRA 52C support a diverse animal community. Grasshopper species can significantly impact plant production during outbreaks or periods of drought, competing with other grazers on this site (Branson and Sword, 2010). Grasshopper density and species richness can increase with changes in vegetation structure and composition associated with disturbances such as fire and grazing (Joern, 2005).
Although amphibians use wetlands throughout MLRA 52 for breeding, most amphibian species, including boreal chorus frog (Pseudacris maculata), western tiger salamander (Ambystoma mavortium), and plains spadefoot (Spea bombifrons), rely on the surrounding grasslands for survival during the non-breeding season (Semlitsch, 2000; Mushet et al., 2012). Similarly, several reptile species, including, prairie rattlesnake (Crotalus viridis), gophersnake (Pituophis catenifer), and plains gartersnake (Thamnophis radix) occur throughout grassland communities.
A variety of migratory grassland birds breed throughout this ecological site. Eight bird species that are endemic or restricted to the Northern Great Plains breed in MLRA 52 (Knopf, 1996). The composition of grassland birds varies with vegetation structure, and the species composition of the breeding bird community will vary depending upon the state and/or community phase occurring on the site (Madden et al., 2000; Henderson and Davis, 2014). For example, species such as Sprague’s pipit (Anthus spragueii) and Baird’s sparrow (Ammodramus bairdii) are more abundant in native, mixed-grass communities associated with the Reference State (Madden et al., 2000; Davis et al., 2013). Similarly, species such as McCown’s longspur (Rhynchophanes mccownii) primarily occur in plant communities dominated by shortgrasses (With, 2010). Most endemic grassland songbirds have reduced abundance and nesting success in grasslands that have been planted with non-native, perennial grasses, analogous to the Post-Cropland State (5) (Davis et al., 2013). Other bird species such as long-billed curlew (Numenius americanus) and greater sage grouse (Centrocercus urophasianus) rely on a variety of habitats for nesting and brood-rearing, emphasizing the importance of managing for diverse vegetation structure (Derner et al., 2009).
Upland nesting waterfowl species, including lesser scaup (Aythya affinis), mallard (Anas platyrhynchos), gadwall (Anas strepera), American wigeon (Anas americana), Eurasian teal (Anas crecca), Blue-winged teal (Anas discors), and northern pintail (Anas acuta) require extensive grasslands represented by this ecological site for nesting and brood-rearing (Stephens et al., 2005). Additionally, several raptor species including, the northern harrier (Circus cyaneus), Swainson’s hawk (Buteo swainsoni), and ferruginous hawk (Buteo regalis), as well as the short-eared owl (Asio flammeus) breed in these plant communities.
Rodents such as Richardson’s ground squirrel (Urocitellus richardsonii) and black-tailed prairie dog (Cynomys ludovicianus) play an important role in plant species composition and production through the excavation of soils to create burrows (Bylo et al., 2014). Historically, native ungulate grazers, in conjunction with fire and drought, played an important ecological role in shaping the composition and structure of the plant communities on this site. Historic grazers included bison (Bison bison), elk (Cervus elaphus), deer (Odocoileus spp.), and pronghorn (Antilocapra americana) (Knopf and Samson, 1997). Cattle have largely replaced these species as the dominant grazer of this site.Hydrological functions
The primary limitation to infiltration on this site is soil structure. While infiltration is generally high in the surface horizon, the underlying natric horizon one to four inches below the surface severely restricts infiltration and root growth, thus favoring the shallow-rooted rhizomatous grasses. While soil erosion is typically minimal, during heavy precipitation events, water may run off the site if it is in a micro-high position or conversely onto the site if it is in a micro-low position.
Recreational uses
This ecological site offers fair to good opportunities for nature observation, photography, and hunting.
Wood products
This ecological site has little to no potential for wood products.
Other products
This ecological site is suitable for grazing by cattle. Due to the hardpan nature of these soils, this ecological site is not well suited for cropland. However, despite the soil limitations and relatively low crop yields this site has been broken and managed as cropland in places.
Other information
For plant preferences by animal kind refer to: Field Office Technical Guide, Section II, Ecological Site Descriptions, General Information.
Supporting information
Inventory data references
A minimum of 20 low or medium observations are required to meet verification level status. This ESD is citing National Resources Inventory (NRI) and 417 data to meet these minimums. Individual observations are listed in EDIT and are viewable behind the login. A corresponding tracking sheet is available in the MLRA office that links the list to the actual observations used in the analysis. A total of 29 plots ranging from low to high intensity were used as a basis for this ecological site. Plant community data are based primarily on high-intensity data collected at five plots representing the Rhizomatous Wheatgrass Plant community (1.1). Vegetation data collection protocols followed (Herrick et al., 2009).
Other references
References cited in this ecological site description include:
Adams, B. W., J. Richman, L. Poulin-Klein, K. France, D. Moisey, and R. L. McNeil. 2013. Rangeland plant communities for the dry mixed grass natural subregion of Alberta. Second approximation. Rangeland management branch, policy division, Alberta Environment and Sustainable Resource Development, Lethbridge, Pub. No. T/040 135pp.
Anderson, R. C. 2006. Evolution and origin of the central grassland of North America: climate, fire, and mammalian grazers. 133:626-647.
Baskin, J. M., and C. C. Baskin. 1981. Ecology of germination and flowering in the weedy winter annual grass Bromus japonicus. Journal of Range Management 34:369-372.
Biondini, M. E., and L. Manske. 1996. Grazing frequency and ecosystem processes in a northern mixed prairie, USA. Ecological Applications 6:239-256.
Biondini, M. E., B. D. Patton, and P. E. Nyren. 1998. Grazing intensity and ecosystem processes in a northern mixed-grass prairie, USA. Ecological Applications 8:469-479.
Bragg, T.B., 1995. The physical environment of the Great Plains grasslands. In: Joern, A., Keeler, K.H. (Eds.), The Changing Prairie. Oxford University Press, Oxford, pp. 49–81.
Branson, D. H., and G. A. Sword. 2010. An experimental analysis of grasshopper community responses to fire and livestock grazing in a northern mixed-grass prairie. Environmental Entomology. 39:1441-1446.
Bylo, L. N., N. Koper, and K. A. Molloy. 2014. Grazing intensity influences ground squirrel and American badger habitat use in mixed-grass prairies. Rangeland Ecology and Management 67:247-254.
Christian, J. M., and S. D. Wilson. 1999. Long-term ecosystem impacts of an introduced grass in the Northern Great Plains. Ecology. 80:2397-2407.
Clarke, S.E, E.W. Tisdale, and N.A. Skoglund. 1947. The effects of climate and grazing practices on short-grass prairie vegetation in southern Alberta and southwestern Saskatchewan. Canadian Department of Agriculture Technical Bulletin No. 46
Cleland, D.T.; Avers, P.E.; McNab, W.H.; Jensen, M.E.; Bailey, R.G., King, T.; Russell, W.E. 1997. National Hierarchical Framework of Ecological Units. Published in, Boyce, M. S.; Haney, A., ed. 1997. Ecosystem Management Applications for Sustainable Forest and Wildlife Resources. Yale University Press, New Haven, CT.
Cooper, S. V., C. Jean, and P. Hendricks. 2001. Biological survey of a prairie landscape in Montana’s glaciated plains. Report to the Bureau of Land Management. Montana Natural Heritage Program, Helena. 24 pp. plus appendices.
Coupland, R. T. 1950. Ecology of the mixed prairie of Canada. Ecological Monographs 20:271-315.
Coupland, R. T. 1958. The effects of fluctuations in weather upon the grasslands of the Great Plains. Botanical Review 24:273-317.
Coupland, R. T. 1961. A reconsideration of grassland classification in the Northern Great Plains of North America. Journal of Ecology 49:135-167.
Coupland, R.T., and R. E. Johnson. 1965. Rooting characteristics of native grassland species in Saskatchewan. The Journal of Ecology 53:475-507.
Davis, S. K., R. J. Fisher, S. L. Skinner, T. L. Shaffer, and R. M. Brigham. 2013. Songbird abundance in native and planted grassland varies with type and amount of grassland in the surrounding landscape. The Journal of Wildlife Management 77:908-919.
DeLuca, T. H., and P. Lesica. 1996. Long-term harmful effects of crested wheatgrass on Great Plains grassland ecosystems. Journal of Soil and Water Conservation 51: 408-409.
Derner, J. D., and R. H. Hart. 2007. Grazing-induced modifications to peak standing crop in northern mixed-grass prairie. Rangeland Ecology and Management 60:270-276.
Derner, J. D., and A. J. Whitman. 2009. Plant interspaces resulting from contrasting grazing management in northern mixed-grass prairie: implications for ecosystem function. Rangeland Ecology and Management 62:83-88.
Derner, J. D., W. K. Lauenroth, P. Stapp, and D. J. Augustine. 2009. Livestock as ecosystem engineers for grassland bird habitat in the western Great Plains of North America. Rangeland Ecology and Management 62:111-118.
Dix, R. L. 1960. The effects of burning on the mulch structure and species composition of grasslands in western North Dakota. Ecology 41:49-56.
Dormaar, J. F., and S. Smoliak. 1985. Recovery of vegetative cover and soil organic matter during revegetation of abandoned farmland in a semiarid climate. Journal of Range Management 38:487-491.
Dormaar, J. F., and W. D. Willms. 1990. Effect of grazing and cultivation on some chemical properties of soils in the mixed prairie. Journal of Range Management 43:456-460.
Dormaar, J. F., B. W. Adams, and W. D. Willms. 1994. Effect of grazing and abandoned cultivation on a Stipa-Bouteloua community. Journal of Range Management 47:28-32.
Dormaar, J. F., M. A. Naeth, W. D. Willms, and D. S. Chanasyk. 1995. Effect of native prairie, crested wheatgrass (Agropyron cristatum) and Russian wildrye (Elymus junceus) on soil chemical properties. Journal of Range Management 48:258-263.
Fansler, V. A., and J. M. Mangold. 2010. Restoring native plants to crested wheatgrass stands. Restoration Ecology 19:16-23.
Fullerton, D.S. and R.B. Colton. 1986. Stratigraphy and Correlation of the Glacial Deposits on the Montana Plains. U.S. Geological Survey.
Fullerton, D.S., R.B. Colton, C.A. Bush, and A.W. Straub. 2004. Map showing spatial and temporal relations of mountain and continental glaciations on the northern plains, primarily in northern Montana and northwestern North Dakota. U.S. Geologic Survey pamphlet accompanying Scientific Investigations Map 2843.
Fullerton, D.S., R.B. Colton, and C.A. Bush. 2013, Quaternary geologic map of the Shelby 1° x 2° quadrangle, Montana: U.S. Geological Survey Open-File Report 2012–1170, scale 1:250,000
Haferkamp, M. R., R. K. Heitschmidt, and M. G. Karl. 1997. Influence of Japanese brome on western wheatgrass yield. Journal of Range Management 50:44-50.
Harmoney, K. R. 2007. Grazing and burning Japanese brome (Bromus japonicus) on mixed grass rangelands. Rangeland Ecology and Management 60:479-486.
Hart, M., S. S. Waller, S. R. Lowry, and R. N. Gates. 1985. Disking and seeding effects on sod bound mixed prairie. Journal of Range Management 38:121-125.
Heidinga, L., and S. D. Wilson. 2002. The impact of an invading alien grass (Agropyron cristatum) on species turnover in native prairie. Diversity and Distributions 8:249-258.
Heitschmidt, R. K., and L. T. Vermeire. 2005. An ecological and economic risk avoidance drought management decision support system. In: J.A. Milne (ed.) Pastoral systems in marginal environments. XXth International Grasslands Congress. July 2005. p. 178.
Henderson, A. E., and S. K. Davis. 2014. Rangeland health assessment: a useful tool for linking range management and grassland bird conservation? Rangeland Ecology and Management 67:88-98.
Henderson, D. C., and M. A. Naeth. 2005. Multi-scale impacts of crested wheatgrass invasion in mixed-grass prairie. Biological Invasions 7:639-650.
Herrick, J.E., J.W. Van Zee, K.M. Havstad, L.M. Burkett, and W.G. Whitford. 2009. Monitoring manual for grassland, shrubland and savanna ecosystems. U.S. Department of Agriculture, Agricultural Research Service, Jornada Experimental Range, Las Cruces, NM.
Higgins, K. F. 1986. Interpretation and compendium of historical fire accounts in the Northern Great Plains. U.S. Fish and Wildlife Service Resource Publication 161, Washington, DC.
Holechek, J. L. 1981. Crested wheatgrass. Rangelands 3:151-153.
Joern, A. 2005. Disturbance by fire frequency and bison grazing modulate grasshopper assemblages in tallgrass prairie. Ecology 86:861-873.
Knopf, F. L. 1996. Prairie legacies-birds. Pp. 135-148. In: F. B. Samson and F. L. Knopf (eds.) Prairie conservation: preserving North America’s most endangered ecosystem. Island Press, Washington, DC.
Knopf, F. L., and F. B. Samson. 1997. Conservation of grassland vertebrates. Pp. 273-289. In: F. B. Samson and F. L. Knopf (eds.) Ecology and conservation of Great Plains vertebrates: Ecological Studies 125. Springer-Verlag, New York, NY.
Krzic, M., K. Broersma, D. J. Thompson, and A. A. Bomke. 2000. Soil properties and species diversity of grazed crested wheatgrass and native rangelands. Journal of Range Management 53:353-358.
Lacey, J., R. Carlstrom, and K. Williams. 1995. Chiseling rangeland in Montana. Rangelands 17:164-166.
Lauenroth, W. K., O. E. Sala, D. P. Coffin, and T. B. Kirchner. 1994. The importance of soil water in recruitment of Bouteloua gracilis in the shortgrass steppe. Ecological Applications 4:741-749.
Laycock, W. A. 1988. History of grassland plowing and grass planting on the Great Plains. In: J. E. Mitchell (ed.) Impacts of the Conservation Reserve Program in the Great Plains: symposium proceedings, September 16-18, 1987. USDA, General Technical Report RM-158. Rocky Mountain Forest and Range Experiment Station, Fort Collins, Colorado.
Laycock, W. A. 1991. Stable states and thresholds of range condition on North American rangelands. Journal of Range Management 44:427-433.
Lockwood, J. A. 2004. Locust: the devastating rise and mysterious disappearance of the insect that shaped the American frontier. Basic Books. New York, NY.
Looman, J., and D. H. Heinrichs. 1973. Stability of crested wheatgrass pastures under long-term pasture use. Canadian Journal of Plant Science 53:501-506.
Madden, E. M., R. K. Murphy, A. J. Hansen, and L. Murray. 2000. Models for guiding management of prairie bird habitat in northwestern North Dakota. The American Midland Naturalist 144:377-392.
McNab, W.H.; Cleland, D.T.; Freeouf, J.A.; Keys, Jr., J.E.; Nowacki, G.J.; Carpenter, C.A., comps. 2007. Description of ecological subregions: sections of the conterminous United States [CD-ROM]. Gen. Tech. Report WO-76B. Washington, DC: U.S. Department of Agriculture, Forest Service. 80 p.
Miller, J. J. and J. A. Brierley. 2011. Solonetzic soils of Canada: genesis, distribution, and classification. Canadian Journal of Soil Science 91:889-902.
Montana State College. 1949. Similar Vegetative Rangeland Types in Montana. Montana State College, Agri. Exp. Station. 35 p.
Mushet, D. M., N. H. Euliss, Jr., and C. A. Stockwell. 2012. A conceptual model to facilitate amphibian conservation in the Northern Great Plains. Great Plains Research 22:45-58.
Nesser, John A.; Ford, Gary L.; Maynard, C. Lee; Page-Dumroese, Deborah S. 1997. Ecological units of the Northern Region: Subsections. Gen. Tech. Rep. INT-GTR-369. Ogden, UT: U.S. Department of Agriculture, Forest Service, Intermountain Research Station. 88 p.
Oard, M. J. A method of predicting Chinook winds east of the Montana Rockies. 1993. Weather and Forecasting 8:166-180
Ogle, D., L. St. John, J. Cornwell, L. Holzworth, M. Majerus, D. Tober K. Jensen, K. Sanders Ed. (rev) St. John, 2012. Plant guide for Russian wildrye (Psathyrostachys junceus). USDA-Natural Resources Conservation Service, Aberdeen Plant Materials Center. Aberdeen, Idaho 83210.
Ogle, S. M., W. A. Reiners, and K. G. Gerow. 2003. Impacts of exotic annual brome grasses (Bromus spp.) on ecosystem properties of the northern mixed grass prairie. American Midland Naturalist 149:46-58.
Roath, L. R. 1988. Implications of land conversions and management for the future. In: J. E. Mitchell (ed.) Impacts of the Conservation Reserve Program in the Great Plains: symposium proceedings, September 16-18, 1987. USDA, General Technical Report RM-158. Rocky Mountain Forest and Range Experiment Station, Fort Collins, Colorado.
Rogler, G. A., and R. J. Lorenz. 1983. Crested wheatgrass: early history in the United States. Journal of Range Management 36:91-93.
Romo, J. T. and Y. Bai. 2004. Seed bank and plant community composition, Mixed Prairie of Saskatchewan. Journal of Range Management 57: 300-304
Romo, J. T. 2011. Clubmoss, precipitation, and microsite effects on emergence of graminoid and forb seedlings in the semiarid northern mixed prairie of North America. Journal of Arid Environments 75:98-105.
Rowe, J. S. 1969. Lightning fires in Saskatchewan grassland. The Canadian Field Naturalist 83:317-327.
Salo, E. D., K. F. Higgins, B. D. Patton, K. K. Bakker, W. T. Barker, B. Kreft, and P. E. Nyren. 2004. Grazing intensity effects on vegetation, livestock and non-game birds in North Dakota mixed-grass prairie. Proceedings of the 19th North American Prairie Conference, Madison, Wisconsin.
Samuel, M. J., and R. H. Hart. 1994. Sixty-one years of secondary succession on rangelands of the Wyoming High Plains. Journal of Range Management 47:184-191.
Semlitsch, R. D. 2000. Principles for management of aquatic-breeding amphibians. The Journal of Wildlife Management 64:615-631.
Shay, J., D. Kunec, and B. Dyck. 2001. Short-term effects of fire frequency on vegetation composition and biomass in mixed prairie in south-western Manitoba. Plant Ecology 155:157-167.
Smith, B., and G. J. McDermid. 2014. Examination of fire-related succession within the dry mixed-grass subregion of Alberta with the use of MODIS and Landsat. Rangeland Ecology and Management 67:307-317.
Smith, R. E. 2013. Conserving Montana’s sagebrush highway: long distance migration in sage-grouse. M.S. Thesis. University of Montana, Missoula.
Smoliak, S., J. F. Dormaar, and A. Johnston. 1972. Journal of Range Management 25:246-250.
Smoliak, S. 1974. Range vegetation and sheep production at three stocking rates on Stipa-Bouteloua prairie. Journal of Range Management 27:23-26.
Smoliak, S., and J. F. Dormaar. 1985. Productivity of Russian wildrye and crested wheatgrass and their effect on prairie soils. Journal of Range Management 38:403-405.
Soil Survey Staff. 2014. Keys to Soil Taxonomy, 12th ed. USDA-Natural Resources Conservation Service, Washington, DC.
Soller, D.R 2001. Map showing the thickness and character of Quaternary sediments in the glaciated United States east of the Rocky Mountains. U.S. Geological Survey Miscellaneous Investigations Series I-1970-E, scale 1:3,500,000
Stephens, S. E., J. J. Rotella, M. S. Lindberg, M. L. Taper, and J. K. Ringelman. 2005. Duck nest survival in the Missouri Coteau of North Dakota: landscape effects at multiple spatial scales. Ecological Applications 15:2137-2149.
Umbanhowar, Jr., C. E. 2004. Interactions of climate and fire at two sites in the Northern Great Plains. Palaeogeography, Palaeoclimatology, and Palaeoecology 208:141-152.
U.S. Fish and Wildlife Service. 2013. Greater sage-grouse (Centrocercus urophasianus)
conservation objectives: Final Report. U.S. Fish and Wildlife Service.
Van Dyne, G. M., and W. G. Vogel. 1967. Relation of Selaginella densa to site, grazing, and climate. Ecology 48:438-444.
Vaness, B. M., and S. D. Wilson. 2007. Impact and management of crested wheatgrass (Agropyron cristatum) in the northern Great Plains. Canadian Journal of Plant Science 87:1023-1028.
Vuke, S.M., K. W. Porter, J. D. Lonn, and D.A. Lopez. 2007. Geologic Map of Montana - Information Booklet: Montana Bureau of Mines and Geology Geologic Map 62-D.
Whisenant, S. G. 1990. Postfire population dynamics of Bromus japonicus. American Midland Naturalist 123:301-308.
Wilson, S. D., and J. M. Shay. 1990. Competition, fire, and nutrients in a mixed-grass prairie. Ecology 71:1959-1967.
With, K. A. 2010. McCown's Longspur (Rhynchophanes mccownii), The Birds of North America Online (A. Poole, Ed.). Ithaca: Cornell Lab of Ornithology; Retrieved from the Birds of North America Online: http://bna.birds.cornell.edu/bna/species/09Contributors
Karen Newlon
Scott Brady
Stuart VeithApproval
Kirt Walstad, 5/08/2025
Acknowledgments
A number of USDA-NRCS and partner staff supported this project. Staff contributions are as follows: Field Data Collection Montana Natural Heritage Program (MTNHP) GIS Products, Data Summaries, Contract Liaison Cathy Maynard, USDA-NRCS (retired) Background Research and Literature Review Karen Newlon, formerly MTNHP Scott Brady, USDA-NRCS Soil Concepts, Soils Information, and Field Descriptions Charlie French, USDA-NRCS (retired) Stuart Veith, USDA-NRCS Josh Sorlie, USDI-BLM Jack Robertson, formerly USDA-NRCS NASIS Reports, Data Exports, and Soil Sorts Bill Drummond, USDA-NRCS (retired) Peer Review and Beta Testing Kirt Walstad, USDA-NRCS Jon Siddoway, USDA-NRCS (retired) Rick Caquelin, USDA-NRCS (retired) Malta Field Office, USDI-BLM Havre Field Office, USDI-BLM Quality Control Grant Peterson, USDA-NRCS Quality Assurance Kirt Walstad, USDA-NRCS Preceding Version(s): Claypan 10 to 14 inch p.z. R052XC204MT (Lacey et al., 2005) Claypan 10 to 14 inch p.z. R052XN204MT (Lacey et al., 2005) Thin Claypan Dry Grassland V 1.0 R052XY165MT (Newlon et al., 2018)
Rangeland health reference sheet
Interpreting Indicators of Rangeland Health is a qualitative assessment protocol used to determine ecosystem condition based on benchmark characteristics described in the Reference Sheet. A suite of 17 (or more) indicators are typically considered in an assessment. The ecological site(s) representative of an assessment location must be known prior to applying the protocol and must be verified based on soils and climate. Current plant community cannot be used to identify the ecological site.
Author(s)/participant(s) Scott Brady, Karen Newlon Contact for lead author 206 25th Ave. West Havre, MT 59501 Date 04/09/2024 Approved by Approval date Composition (Indicators 10 and 12) based on Foliar Cover Indicators
-
Number and extent of rills:
Rills are typically not present in the reference condition. Slight evidence of rills may occur following a rainfall event, but rills would be short (less than 3 feet) and discontinuous. -
Presence of water flow patterns:
Water flow patterns are typically not present in the reference condition. If present, they are most likely to occur on the margins of the site or where root mats have been disturbed. They are typically faint, disconnected, and very short in length (less than 1 foot). Slight evidence of water flow patterns may also occur following a rainfall or winter thaw event. -
Number and height of erosional pedestals or terracettes:
Pedestals are rare in the reference condition and are most likely to occur at the margins of the site. If present, they occur on less than 5 percent of plants and are less than ½ inch in height. -
Bare ground from Ecological Site Description or other studies (rock, litter, lichen, moss, plant canopy are not bare ground):
Bare ground is typically less than 10 percent. It typically consists of randomly scattered patches less than 2 inches in diameter, particularly where clubmoss is absent or disturbed. Note: Indicator should be evaluated in the context of current years climate and disturbance patterns. Events such as drought, hail, fire, etc. may increase bare ground. Bare ground is defined as exposed mineral soil without cover from vegetation, litter, surface fragments, or biotic crust (measured by Line-Point Intercept method). -
Number of gullies and erosion associated with gullies:
Active gullies are not present in the reference state. If there is evidence of past erosion that has created gullies, these areas should have stable vegetative cover and no active erosion is evident. -
Extent of wind scoured, blowouts and/or depositional areas:
Wind scoured or depositional areas are rare in the reference condition. If present, they occur on less than 5 percent of the area and tend to be inconspicuous and not connected. -
Amount of litter movement (describe size and distance expected to travel):
Litter movement is typically not evident in the reference condition. If present, fine litter movement is typically less than 1 foot and limited to within water flow patterns, with little or no accumulation around obstructions. Large litter movement is not evident. -
Soil surface (top few mm) resistance to erosion (stability values are averages - most sites will show a range of values):
The average soil stability rating is 5 to 6, both under plant canopies and in plant interspaces. -
Soil surface structure and SOM content (include type of structure and A-horizon color and thickness):
Due to natural soil forming processes, soils on this site typically have a thin, loamy surface horizon with a dense, root restricting clay layer underneath. The soil surface horizon averages 2.5 inches (7 cm) thick but may vary from 1.5 to 4 inches (4 to 10 cm) thick. It has thin platy structure, and moist color typically varies from brown (10YR 5/3) to dark grayish brown (10YR 4/2). The subsurface horizon is hard, clayey, and has columnar structure. -
Effect of community phase composition (relative proportion of different functional groups) and spatial distribution on infiltration and runoff:
Infiltration and runoff on this site is largely controlled by soil properties. Canopy cover of 40 to 75 percent reduces raindrop impact, slows overland flow, and increases time for infiltration into the soil surface horizon. Plant community composition is dominated by mid-statured cool season rhizomatous grasses (25 to 65 percent) with up to 5 percent mid-statured cool season bunchgrasses, which all have root systems that stabilize soil structure and aid infiltration. Infiltration below the surface horizon is severely limited by the dense, clayey subsoil regardless of plant community composition. -
Presence and thickness of compaction layer (usually none; describe soil profile features which may be mistaken for compaction on this site):
A compaction layer is not present in the reference condition; however, the natural soil structure may be confused with a compaction layer. Due to the unique soil forming processes on this site soil structure in the surface horizon is typically thin platy. The subsurface horizon has columnar structure, is hard, and is root restrictive. This hard layer occurs due to natural soil forming processes. -
Functional/Structural Groups (list in order of descending dominance by above-ground annual-production or live foliar cover using symbols: >>, >, = to indicate much greater than, greater than, and equal to):
Dominant:
Typically, cool-season rhizomatous wheatgrasses are the dominant functional/structural group with a combined cover ranging from 25 to 65 percent.Sub-dominant:
Shortgrasses are a subdominant component with 5 to 25 percent cover.Other:
Mid-statured cool season bunchgrasses, forbs, and shrubs/subshrubs are minor components with 0 to 5 percent, 1 to 10 percent, and 5 percent or less cover respectively.Additional:
Functional and structural groups must be evaluated in the context of the current years climate. Climatic fluctuations such as amount and timing of precipitation, temperature, and stored soil moisture may effect composition and structure on the site. -
Amount of plant mortality and decadence (include which functional groups are expected to show mortality or decadence):
Mortality is not evident on rhizomatous herbaceous species. Bunchgrasses may show some signs of dead or dying plant parts, but mortality typically does not exceed 5 percent for any given species. Mortality on woody species is typically 5 percent or less per species. -
Average percent litter cover (%) and depth ( in):
Total litter cover averages about 35 percent but may range from 20 to 50 percent depending productivity and grazing use. This includes all detached plant material, both on the soil surface and suspended in the canopy. Most litter is loosely distributed throughout the canopy and it is estimated that only 5 to 10 percent is in contact with the soil surface. It does not typically accumulate to a measurable depth on the soil surface. Note: Indicator should be evaluated in the context of current years climate and disturbance patterns. Above average precipitation may increase litter amounts whereas events such as drought, hail, fire, etc. may decrease litter amounts. -
Expected annual annual-production (this is TOTAL above-ground annual-production, not just forage annual-production):
Total annual production is strongly influenced by climatic factors such as amount and timing of precipitation, temperature, and stored soil moisture and must be evaluated within the context of the current climatic conditions. Estimated annual production expected on this site for below average, average, and above average years is as follows: Below Average (pounds per acre) Grasses: 220 to 370 Forbs: 40 to 65 Shrubs: 10 to 15 Total: 270 to 450 Average (pounds per acre) Grasses: 325 to 490 Forbs: 60 to 90 Shrubs: 15 to 20 Total: 400 to 600 Above Average (pounds per acre) Grasses: 410 to 620 Forbs: 75 to 115 Shrubs: 15 to 25 Total: 500 to 760 -
Potential invasive (including noxious) species (native and non-native). List species which BOTH characterize degraded states and have the potential to become a dominant or co-dominant species on the ecological site if their future establishment and growth is not actively controlled by management interventions. Species that become dominant for only one to several years (e.g., short-term response to drought or wildfire) are not invasive plants. Note that unlike other indicators, we are describing what is NOT expected in the reference state for the ecological site:
Potential invasive plants on this site are crested wheatgrass, noxious weeds, and annual bromes. Invasive species are typically absent or constitute less than 5 percent cover in the reference condition. However, annual brome species such as field brome (<a class="species-link" href="https://plants.usda.gov/core/profile?symbol=BRAR5" target="_blank" title="Open in plants.usda.gov"><i>Bromus arvensis</i></a>) may exhibit seasonal abundance, depending on moisture and germination conditions, which result in short-term departures from reference. -
Perennial plant reproductive capability:
In the reference condition, all plants are vigorous enough for reproduction either by seed or tillers. For grasses and forbs: at least 50 percent of plants are capable of producing seedheads. For shrubs: 50 percent or more of plants are capable of producing flowering leaders. Note: Must be evaluated in the context of the current years climate. Climatic fluctuations such as amount and timing of precipitation, temperature, and stored soil moisture may effect flower or seed production depending on the particular species.
Print Options
Sections
Font
AAAAOther
PrintThe Ecosystem Dynamics Interpretive Tool is an information system framework developed by the USDA-ARS Jornada Experimental Range, USDA Natural Resources Conservation Service, and New Mexico State University.
Accessibility statement


