
Natural Resources
Conservation Service
-
Search


Major Land Resource Area or ecological site by name and/or ID.
PreviousSectionsNextGeneral information
Draft. A draft ecological site description is either incomplete or has not undergone quality control and quality assurance review.
MLRA notes
Major Land Resource Area (MLRA): 022A–Sierra Nevada and Tehachapi Mountains
Major Land Resource Area 22A, Sierra Nevada Mountains, is located predominantly in California and a small section of western Nevada. The area lies completely within the Sierra Nevada Section of the Cascade-Sierra Mountains Province. The Sierra Nevada range is highly asymmetrical with a long, gentle western slope, and a very abrupt eastern slope. The Sierra Nevada consists of hilly to steep mountains and occasional flatter mountain valleys. Elevation ranges between 1,500 and 9,000 ft throughout most of the range, but certain peaks often exceed 12,000 ft. The highest point in the continental US occurs in this MLRA (Mount Whitney, 14,494 ft). Most of the Sierra Nevada is dominated by granitic rock of the Mesozoic age, known as the Sierra Nevada Batholith. The northern half is flanked on the west by a metamorphic belt, which consists of highly metamorphosed sedimentary and volcanic rocks of Paleozoic and Mesozoic ages. Additionally, glacial activity of the Pleistocene has played a major role in shaping Sierra Nevada features, including cirques, arêtes, and glacial deposits and moraines. Average annual precipitation ranges from 20 to 80 inches in most of the area, with increases along elevational and south-north gradients. Soil temperature regime ranges from mesic, frigid, and cryic. Due to the extreme elevational range found within this MLRA, Land Resource Units (LRUs) were designated to group the MLRA into similar land units.
LRU "A" alpine
This LRU occurs at the highest elevations of the Sierra Nevada, above treeline on upper mountain slopes, exposed ridges and mountain peaks. This LRU begins at the alpine treeline ecotone, which occurs at approximately 11,000 feet in the south and central areas and approximately 9,800 feet in the north, and extends up to 14,494 feet (Mount Whitney). Mean annual air temperature (MAAT) ranges from 29 to 35 degrees F, mean annual precipitation (MAP) ranges from 20 to 60 inches, and the frost free season is 20 to 30 days.
Classification relationships
Mediterranean California Alpine Fell-Field (NaturServe 2014).
Sierra Nevada Fell-Field, Holland type 91120 (Holland 1986).Ecological site concept
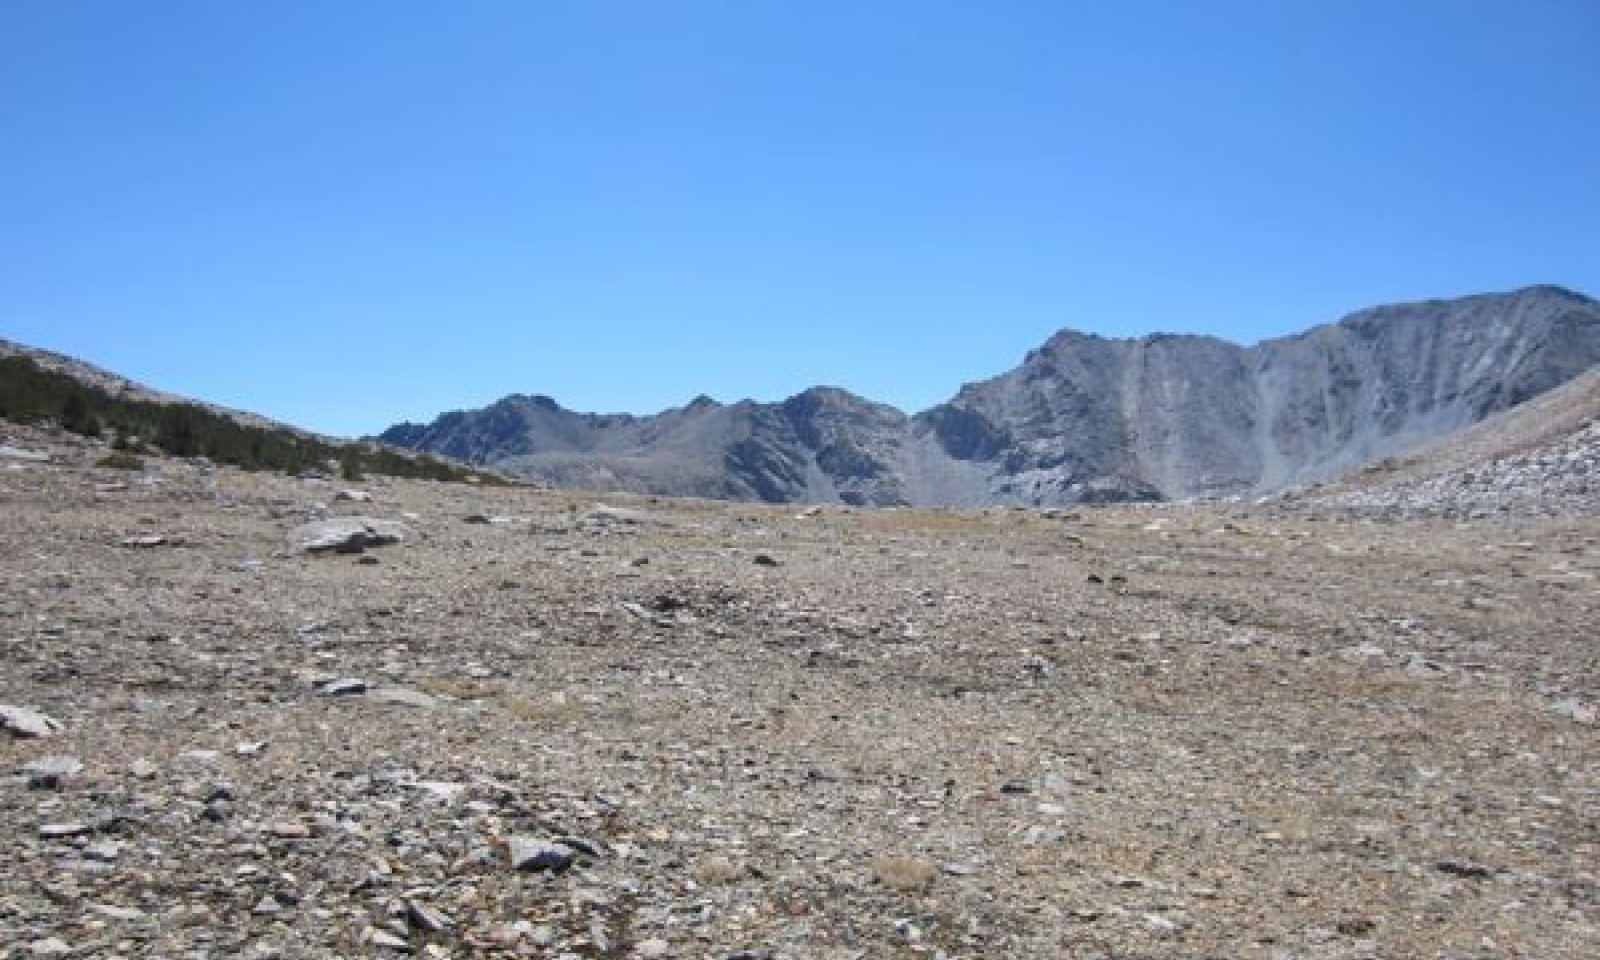
This ecological site occurs on high elevation mountain passes with deep to very deep loamy-skeletal soils derived from glacial till. Strong winds that are funneled through the pass redistribute snow from these areas, creating dry, exposed, extremely cold environments in winter, and droughty environments in summer. These dry windy conditions, cold temperatures, intense solar radiation and a short growing season limit productivity in this ecological site. The vegetation of this site is a fell-field community of low growing subshrubs, forbs and grasses. Species characteristic of dry rocky conditions dominate. However, loamy deep soils have higher water holding capacity than shallow soils found on adjacent ridges, allowing for species characteristic of more mesic conditions, and leading to a diverse plant community. These mesic species are often found in microsites where snow accumulates, such as in the lee of boulders or stones, or depressions in the soil. Sierra mousetail (Ivesia santolinoides) and spreading phlox (Phlox diffusa) dominate.
Table 1. Dominant plant species
Tree Not specified
Shrub Not specified
Herbaceous (1) Ivesia santolinoides
(2) Phlox diffusaPhysiographic features
This site occurs on alpine saddles (passes). Slopes range from - to – percent. Elevations are range from - to - feet. Runoff class is - to -.
Table 2. Representative physiographic features
Landforms (1) Saddle
(2) Mountain
Climatic features
The climate of this ecological site is characterized by cool temperatures, wet winters with most precipitation falling as snow in winters, and relatively dry summers. The mean annual precipitation ranges from - to - inches. The mean annual temperature ranges from - to - degrees F. The frost-free (>32F) season is - to – days. The freeze-free (>28F) season is - to - days.
Table 3 Representative climatic features
Frost-free period (average) 0 days Freeze-free period (average) 0 days Precipitation total (average) 0 in BarLineFigure 1. Monthly precipitation range
BarLineFigure 2. Monthly average minimum and maximum temperature
Figure 3. Annual precipitation pattern
Figure 4 Annual average temperature pattern
">Influencing water features
Soil features
The soils associated with this ecological site are deep to very deep, and formed in glacial till. They are -- drained with -- permeability. The soil moisture regime is xeric and the soil temperature regime is cryic. Surface rock fragments smaller than 3 mm in diameter range from -- to -- percent cover, and larger fragments range from -- to -- percent. Surface textures are --. Subsurface textures are --. Subsurface rock fragments smaller than 3 mm in diameter range from -- to -- percent by volume, and larger fragments range from -- to -- percent (for a depth of - to -- inches). The -- soils are correlated to this ecological site. The -- soils are (Loamy skeletal typic cryorthents).
This ecological site has been correlated with the following mapunits and soil components in the Sequoia and Kings Canyon National Parks soil survey area (CA792):
Area_sym ; Musym ; MUname ; Compname ; Local_phase ; Comp_pct
Ecological dynamics
Abiotic factors
This ecological site occurs on high elevation mountain passes with deep to very deep loamy-skeletal soils derived from glacial till. Strong winds that are funneled through the pass redistribute snow from these areas, creating dry, exposed, extremely cold environments in winter, and droughty environments in summer. These dry windy conditions, cold temperatures, intense solar radiation and a short growing season limit productivity in this ecological site, promoting fell-field communities of low growing subshrubs, forbs and grasses. Species characteristic of dry rocky conditions dominate. However, loamy deep soils have higher water holding capacity than shallow soils found on adjacent ridges, allowing for species characteristic of more mesic conditions, and leading to a diverse plant community. These mesic species, for example alpine gentian(Gentiana newberryi) and Idaho bentgrass (Agrostis idahoensis) are often found in microsites where snow accumulates, such as in the lee of boulders or stones, or depressions in the soil. Sierra mousetail (Ivesia santolinoides) and spreading phlox (Phlox diffusa) dominate.
Alpine plant communities are determined by a snow cover gradient that is the product of wind exposure and topography, and by soils and geologic substrate (Billings and Mooney 1968, Burns and Tonkin 1982, Seastedt et al. 2004). Areas with exposed topography, especially with aspects that are exposed to prevailing winds, are blown free of snow for the majority of the year, for example periods of 225 or more snow-free days/year (Billings and Mooney 1968) are common. Wind through mountain passes can be extreme due to the funneling ‘Bernoulli effect’, as wind seeks a way around higher peaks on either side of the pass. These windblown sites support a fell-field community that is largely covered in surface rock fragments, and limited to low-statured, long-lived, slow-growing subshrub, forb and grass species (Smiley 1915, Kilkoff 1965, Billings and Mooney 1968, Körner 2003, Elliot and Jules 2005). These open fell-fields are characterized by a high percentage of surface rock, with sparsely distributed vegetation. Fell-field plants are less insulated than sod-forming meadows, and subject to rapid increases in soil temperature as well as rapid decreases (Billings and Mooney 1968). Subshrubs such as spreading phlox and cushion buckwheat (Eriogonum ovalifolium) are cushion forming, and forbs such as Nuttall’s sandwort (Minuarta nuttallii) and rosy pussytoes (Antennaria rosea) are mat forming, while grasses form tight tussock growth forms (Billings and Mooney 1968, Körner 2003). These adaptations trap heat, which increases photosynthetic capacity in these cold environments, and limits moisture loss due to transpiration (Billings and Mooney 1968, Körner 2003).
Disturbance/Ecological factors
Fluctuations in temperature and moisture are the primary natural disturbance impacting this ecological site, and these may temporarily alter species composition. Global climate change will likely impact this site and is discussed below, but is not included in the state-and-transition model. Anthropogenic disturbances such as trail building and trampling may impact this site, with very slow recovery due to the slow growth rate of species in this harsh environment. Sheep grazing in the late 1800’s and early 1900’s was intense and ubiquitous in the Sierra Nevada (e.g. Ratliff 1974, Vankat and Major, 1978, Benedict 1983, Ratliff 1985, Odion et al. 1988), and may have impacted this site. Impacts could include trampling and compaction of soils, trampling of sensitive vegetation, and alteration of species composition by selective grazing. Data is not available for grazing impacts on this site, and they are not included in the state-and-transition model.
Long periods of severe drought would likely lower diversity on this site, eliminating or greatly reducing species dependent on greater moisture availability. It would also likely lower production and cover overall, as even drought-adapted species may experience leaf dieback or reduce production during drought (e.g. Peterson and Billings 1982). At the time data was collected for this site annual precipitation was 65 percent of average; however, the Sierra Nevada were also in the third year of drought and evidence of dieback was apparent (see photo in community phase 1.2). Very wet years on the other hand are likely to see an increase in moisture dependent plants, and could see dieback in species adapted to dry conditions. Wet conditions caused by an increased duration in the snowpack would shorten the already limited growing season of this ecological site, causing reduced cover and production in the plant community (e.g. Franklin 2013). Wet and warm conditions without an increase in snowpack duration would likely see an increase in productivity and cover (e.g. Franklin 2013, Klimesova et al. 2013).
An ongoing pattern of warming and decreased snowpack is predicted under global climate change scenarios for the Sierra Nevada (e.g Hayhoe et al. 2004, Safford et al. 2012). Recent California based climate models predict a 9 degree F increase in temperature by 2100, and more conservative models predict a 2 to 4 degree F increase in winter and 4 to 8 degree increase in summer (Safford et al. 2012). Models are more variable for precipitation, but recent models for the Sierra Nevada, predict similar to slightly less precipitation. Most models agree that summers will become drier, since more of the precipitation is predicted to come as rain, and snow melt-off will occur earlier in spring (Hayhoe et al. 2004, Safford et al. 2012). Alpine areas have been called bellwethers for global climate change impacts (e.g. Seastedt et al. 2004), due to a highly specialized flora and fauna that may not compete well with a lessening of harsh environmental conditions, and no higher elevations to retreat. However, unidirectional change may not be realistic. Microtopographic variation that allows for xeric and mesic species to co-occur may allow for within site or more local migrations, and confer resilience to climate change (Gibson et al. 2008, Spasojevic et al. 2013). Alternatively fell-field communities adapted to severe drought may expand downward into previously moister locations with increased warming and reduced precipitation (Spasojevic et al. 2013). Long-term studies of fell-field communities in Colorado have shown these dry systems to be fairly resilient to change, with impermanent transitions occurring in response to annual variations in climate (Johnson et al. 2011, Spasojevic et al. 2013). However, while communities are not being lost, there is an overall trend of increased diversity as species from lower elevations move up, and in time, these species may outcompete the locals (Johnson et al. 2011, Spasojevic et al. 2013).
Warmer and drier conditions could lead to an expansion of this ecological site, as it could move into habitats currently occupied by snowbank or moister communities. Warmer temperatures would likely increase the growth and productivity of at least some species in this plant community, for example granite prickly phlox in the eastern Sierra Nevada was shown to have higher growth rates during warmer periods (Franklin 2013). However increasing aridity could offset these increases. Species composition is likely to change; with species that occur in this site but that have a wider ecological amplitude than strictly alpine environments, such as cushion buckwheat (Eriogonum ovalifolium), likely to increase in production and cover. Species richness may increase from species moving upslope, as has already been demonstrated in other alpine environments (e.g. Bahn and Körner 2003, Johnson et al. 2011, Spasojevic et al. 2013). However, these increases in species richness may be offset over time by the extirpation of species that are restricted to the alpine and have no upslope environment to move to, such as rosy buckwheat (Eriogonum rosense) or marumeaf buckwheat (Eriogonum marifolium). A modeling study in the White Mountains of California predicted extinction of 10 out of 14 alpine forbs modeled with a 6 degree temperature increase, with the remaining 4 shrinking to less than 1% of their current range (Van de Ven et al. 2007). A 3 degree warming predicted extinction of 2 species, and severe range restrictions of all others (Van de Ven et al. 2007). Since the specific changes that will occur with global climate change are currently unknown for this site, climate change impacts are not included in the state-and-transition model.
All tabular data listed for a specific community phase within this ecological site description represent a summary of one or more field data collection plots taken in communities within the community phase. Although such data are valuable in understanding the phase (kinds and amounts of ground and surface materials, canopy characteristics, community phase overstory and understory species, production and composition, and growth), it typically does not represent the absolute range of characteristics nor an exhaustive listing of species for all the dynamic communities within each specific community phase.
State and transition model
Custom diagramStandard diagram
Figure 5. R022AA106CA
More interactive model formats are also available. View Interactive Models
More interactive model formats are also available. View Interactive Models
Click on state and transition labels to scroll to the respective textEcosystem states
State 1 submodel, plant communities
State 1
ReferenceCommunity 1.1
Reference
Figure 6. Community phase 1.1

Figure 7. Community phase 1.1
A low statured, low production community dominated by subshrubs and forbs characterizes the reference plant community. Subshrubs and forbs average 32 percent cover, and grasses range from two to 17 percent cover. Rock fragments dominate the soil surface, at 93 percent cover, with gravel sized fragments dominant. Plant cover is often congested, with multiple species growing together in an interwoven mat due to the facilitating effects of established plants (e.g. Billings and Mooney 1968, Greenlee and Calloway 1996). Species richness in this site is high, with an average of 18 species occurring in a given location. Subshrubs characteristic of dry rocky and sandy habitats are prevalent, with spreading phlox, rosy buckwheat, cushion buckwheat, frosted buckwheat (Eriogonum incanum), and marumleaf buckwheat common. Sierra mousetail, a California high elevation endemic that occurs in bare sandy habitats (Jepson 1993) is the dominant forb. Other forbs typically found in dry rocky habitats include Nuttal’s sandwort, sicklekeel lupine (Lupinus albicaulis), Watson’s spikemoss (Selaginella watsonii), and stem raillardella (Raillardella scaposa), which occurs from exposed dry sites to wet sites (Jepson 1993). Forbs more characteristic of wet sites include little elephantshead (Pedicularis attolens), Rydberg’s penstemon (Penstemon rydbergii), creeping sibbaldia (Sibbaldia procumbens), and alpine gentian. Grasses and grasslike species include threadleaf sedge (Carex filifolia), which is typically found on dry montane to alpine sites, Parry’s rush (Juncus parryi), which is found on dry to wet habitats, Sierra woodrush (Luzula orestra), which is found in subalpine and alpine meadows and fellfields, Ross’ sedge (Carex rossii), Sandberg bluegrass (Poa secunda), and squirreltail, all of which have a wide distribution, and Idaho bentgrass which is a wet meadow species.
Figure 8. Annual production by plant type (representative values) or group (midpoint values)
Table 4. Annual production by plant type
Plant type Low
(lb/acre)Representative value
(lb/acre)High
(lb/acre)Forb 70 100 120 Grass/Grasslike 20 27 33 Total 90 127 153 Table 5. Soil surface cover
Tree basal cover 0% Shrub/vine/liana basal cover 0% Grass/grasslike basal cover 0-0% Forb basal cover 0-10% Non-vascular plants 0-0% Biological crusts 0% Litter 0% Surface fragments >0.25" and <=3" 70-80% Surface fragments >3" 20-30% Bedrock 0% Water 0% Bare ground 0-10% Table 6. Canopy structure (% cover)
Height Above Ground (ft) Tree Shrub/Vine Grass/
GrasslikeForb <0.5 0-1% 0-4% 3-18% 20-40% >0.5 <= 1 0-1% – 0-18% 0-5% >1 <= 2 0-1% – 0-2% – >2 <= 4.5 0-1% – – – >4.5 <= 13 0-1% – – – >13 <= 40 – – – – >40 <= 80 – – – – >80 <= 120 – – – – >120 – – – – Community 1.2
Drought (Provisional)
Figure 9. Vegetation dieback with drought
This community phase is characterized by severe drought that reduces moisture microclimate availability on this site. These conditions lead to a decline in species diversity due to a reduction in species requiring moist conditions such as little elephantshead, Rydberg’s penstemon, creeping sibbaldia, alpine gentian, and Idaho agrostis. Overall production and cover also decline with leaf and branch dieback of xeric species, and a lack of reproduction.
Community 1.3
Warm, wet (Provisional)This community phase is characterized by a benign climate and an increase in soil moisture. These conditions cause an increase in moisture requiring species, and an overall increase in production and cover.
Community 1.4
Cold, wet (Provisional)This community phase is characterized by cold wet conditions that increase the amount and duration of the snowpack. These conditions reduce the growing season on this site, reducing cover and production. Species requiring moist conditions are likely to increase, while species adapted to dry conditions may experience dieback.
Pathway 1.1a
Community 1.1 to 1.2
Reference
Drought (Provisional)Occurs with ongoing severe drought.
Pathway 1.1b
Community 1.1 to 1.3Occurs with ongoing abnormally wet and warm conditions that increase moisture availability on this site.
Pathway 1.1c
Community 1.1 to 1.4Occurs with ongoing abnormally wet and cold conditions that increase snowpack on this site.
Pathway 1.2a
Community 1.2 to 1.1
Drought (Provisional)
ReferenceThis pathway occurs with a return to average precipitation conditions.
Pathway 1.2c
Community 1.2 to 1.3Occurs with ongoing abnormally wet and warm conditions that increase moisture availability on this site.
Pathway 1.2b
Community 1.2 to 1.4Occurs with ongoing abnormally wet and cold conditions that increase snowpack on this site.
Pathway 1.3a
Community 1.3 to 1.1This pathway occurs with a return to average precipitation conditions.
Pathway 1.3c
Community 1.3 to 1.2Occurs with ongoing severe drought.
Pathway 1.3b
Community 1.3 to 1.4Occurs with ongoing abnormally wet and cold conditions that increase snowpack on this site.
Pathway 1.4a
Community 1.4 to 1.1This pathway occurs with a return to average precipitation conditions.
Pathway 1.4c
Community 1.4 to 1.2Occurs with ongoing severe drought.
Pathway 1.4b
Community 1.4 to 1.3Occurs with ongoing abnormally wet and warm conditions that increase moisture availability on this site.
Additional community tables
Table 7. Community 1.1 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Forb1 Subshrubs 30–45 spreading phlox PHDI3 Phlox diffusa 0–15 0–7 cushion buckwheat EROV Eriogonum ovalifolium 0–15 0–3 rosy buckwheat ERRO Eriogonum rosense 0–10 0–3 frosted buckwheat ERIN9 Eriogonum incanum 0–5 0–2 marumleaf buckwheat ERMA4 Eriogonum marifolium 0–5 0–2 2 Perennial forbs 50–100 Sierra mousetail IVSA2 Ivesia santolinoides 45–75 4–10 Rydberg's penstemon PERY Penstemon rydbergii 0–10 0–2 Watson's spikemoss SEWA2 Selaginella watsonii 1–7 1–10 sicklekeel lupine LUAL3 Lupinus albicaulis 0–5 0–4 rosy pussytoes ANRO2 Antennaria rosea 0–5 0–2 fleabane ERIGE2 Erigeron 0–5 0–2 little elephantshead PEAT Pedicularis attollens 0–5 0–2 stem raillardella RASC2 Raillardella scaposa 0–4 0–3 alpine gentian GENE Gentiana newberryi 0–4 1–2 Mt. Hood pussypaws CIUMU Cistanthe umbellata var. umbellata 0–2 0–1 creeping sibbaldia SIPR Sibbaldia procumbens 0–2 0–1 Nuttall's sandwort MINU4 Minuartia nuttallii 0–2 0–1 owl's-clover ORTHO Orthocarpus 0–2 0–1 Grass/Grasslike3 Grasses/Grasslikes 20–33 threadleaf sedge CAFI Carex filifolia 1–25 1–5 Parry's rush JUPA Juncus parryi 0–18 0–10 Sierra woodrush LUOR4 Luzula orestera 0–5 0–5 Ross' sedge CARO5 Carex rossii 0–4 0–2 Idaho bentgrass AGID Agrostis idahoensis 0–4 0–2 bluegrass POA Poa 0–3 0–1 Sandberg bluegrass POSE Poa secunda 0–2 0–1 squirreltail ELEL5 Elymus elymoides 0–2 0–1 Table 8. Community 1.2 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 9. Community 1.3 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Table 10. Community 1.4 plant community composition
Group Common name Symbol Scientific name Annual production () Foliar cover (%) Interpretations
Animal community
Yellow bellied marmot (Marmota flaviventris), American pika (Ochotona princeps), and Sierra bighorn sheep (Ovis canadensis sierrae) may use this ecological site.
Recreational uses
This is a scenic alpine area with backcountry hiking use.
Supporting information
Inventory data references
High intensity sampling (Caudle et al. 2013) was used to describe this ecological site. Site characteristics such as aspect, slope, elevation and UTMS were recorded for each plot, along with complete species inventory by ocular percent cover. The line-point intercept method was used to measure foliar cover, groundcover, and vegetation structure. At 100 points along a 400-foot step transect, ground cover and intercepted plant species were recorded by height. The first hit method (Herrick et al. 2009) was used to generate the foliar cover values entered in the community phase composition tables. Annual production was estimated using the double-weight sampling method outlined in the National Range and Pasture Handbook and in Sampling Vegetation Attributes (NRCS 2003 and Interagency Technical Reference 1999 pgs. 102 - 115). For herbaceous vegetation, ten 9.6 square foot circular sub-plots were evenly distributed along a 200 foot transect. For woody and larger herbaceous species production was estimated in four 21’X21’ square plots along the same transect. Weight units were collected for each species encountered in the production plots. The number of weight units for each species is then estimated for all plots. Inventory plots: 2013CA7927036 (Type location) 2013CA7929105
Type locality
Location 1: Fresno County, CA UTM zone N UTM northing 4083186 UTM easting 378218 General legal description The type location is found on Sawmill Pass in Kings Canyon National Park. Other references
Bahn, M. and C. Körner. 2003. Recent increases in summit flora caused by warming in the alps. Pages 437-441 Alpine Diversity in Europe Springer, Berlin.
Benedict, N. B. 1983. Plant associations of subalpine meadows, Sequoia National Park, California. Arctic and Alpine Research 15:383-396.
Billings, W. D. and H. A. Mooney. 1968. The ecology of arctic and alpine plants. Biological Reviews 43:481-529.
Burns, S. F. and P. J. Tonkin. 1982. Soil-geomorhpic models and the spatial distribution and development of alpine soils. Pages 25-44 in C. E. Thorn, editor. Space and time in geomorphology. George Allen and Unwin, London.
Caudle, D., H. Sanchez, J. DiBenedetto, C. Talbot, and M. Karl. 2013. Interagency ecological site handbook for rangelands. USDA-NRCS, USDA-FS, DOI-BLM.
Elliot, S. E. and E. S. Jules. 2005. Small-scale community analyses of alpine ridge vegetation in the central Sierra Nevada. Madroño 52:38-45.
Franklin, R. S. 2013. Growth response of the alpine shrub, Linanthus pungens, to snowpack and temperature at a rock glacier site in the eastern Sierra Nevada of California, USA. Quaternary International 310:20-33.
Gibson, A. C., P. W. Rundel, and M. R. Sharifi. 2008. Ecology and ecophysiology of a subalpine fellfield community on Mount Pinos, Southern California. Madroño 55:41-51.
Greenlee, J. T. and R. M. Calloway. 1996. Abiotic stress and the relative importance of interference and facilitation in montane bunchgrass communities in western Montana. The American Naturalist 148:386-396.
Hayhoe, K., D. Cayan, C. B. Field, P. C. Frumhoff, E. P. Mauren, N. L. Miller, S. C. Moser, S. H. Schneider, K. N. Cahill, E. E. Cleland, L. Dale, R. Drapek, R. M. Hanemann, L. S. Kalkstein, J. Lenihan, C. K. Lunch, R. P. Neilson, S. C. Sheridan, and J. H. Verville. 2004. Emissions pathways, climate change, and impacts on California. Proceedings of the National Academy of Sciences 101.
Holland, R.F., 1986. Preliminary descriptions of the terrestrial natural communities of California. State of California, The Resources Agency, Nongame Heritage Program, Dept. Fish & Game, Sacramento, Calif. 156 pp.
Jepson, W. L. 1993. The Jepson manual: higher plants of California. University of California Press, Berkeley, CA.
Johnson, D. R., D. Ebert-May, P. J. Webber, and C. E. Tweedie. 2011. Forecasting alpine vegetation change using repeat sampling and a novel modeling approach. Ambio 40:693-704.
Kilkoff, L. G. 1965. Microenvironmental influence on vegetation pattern near timberline in the central Sierra Nevada. Ecological Monographs 35:187-211.
Klimesova, J., J. Dolezal, and P. St'astna. 2013. Growth of the alpine herb Rumex alpinus over two decades: effect of climate fluctuations and local conditions. Plant Ecology 214:1071-1084.
Körner, C. 2003. Alpine plant life: functional plant ecology of high mountain ecosystems. Springer-Verlag, Berlin, Germany.
NatureServe. 2014. NatureServe Explorer: An online encyclopedia of life [web application]. Version 7.1. NatureServe, Arlington, Virginia. Available http://explorer.natureserve.org. (Accessed: November 29, 2014 ).
Odion, D. C., T. L. Dudley, and C. M. D'Antonio. 1988. Cattle grazing in southeastern Sierran meadows: ecosystem chane and prospects for recovery. Pages 277-292 Plant biology of eastern California. White Mountain Research Station, University of California, Los Angeles.
Peterson, K. M. and W. D. Billings. 1982. Growth of alpine plants under controlled drought. Arctic and Alpine Research 14:189-194.
Ratliff, R. D. 1974. Short-hair sedge--its condition in the high Sierra Nevada of California. Forest Service, US Dept. of Agriculture, Pacific Southwest Forest and Range Experiment Station.
Ratliff, R. D. 1985. Meadows in the Sierra Nevada of California: state of knowledge. United States Department of Agriculture, U.S. Forest Service, Pacific Southwest Forest and Range Experiment Station, Berkeley, CA.
Safford, H. D., M. North, and M. D. Meyer. 2012. Climate change and the relevance of historical forest conditions. Pages 23-45 in M. North, editor. Managing Sierra Forests. U.S. Department of Agriculture, Forest Service, Pacific Southwest Research Station, Albany, CA.
Smiley, F. J. 1915. The alpine and subalpine vegetation of the Lake Tahoe region. Botanical Gazette 59:265-286.
Seastedt, T. R., W. D. Bowman, T. N. Caine, D. McKnight, A. Townsend, and M. W. Williams. 2004. The landscape continuum: a model for high-elevation ecosystems. Bioscience 54:111-121.
Spasojevic, M. J., W. D. Bowman, H. C. Humphries, T. R. Seastedt, and K. N. Suding. 2013. Changes in alpine vegetation over 21 years: Are patterns across a heterogeneous landscape consistent with predictions? Ecosphere 4.
Van de Ven, C. M., S. B. Weiss, and W. G. Ernst. 2007. Plant species ditributions under present conditions and forecasted for warmer climates in an arid mountain range. Eart Interactions 11:1-33.
Vankat, J. L. and J. Major. 1978. Vegetation changes in Sequoia National Park, California. Journal of Biogeography 5:377-402.
Contributors
Dave Evans
Rangeland health reference sheet
Interpreting Indicators of Rangeland Health is a qualitative assessment protocol used to determine ecosystem condition based on benchmark characteristics described in the Reference Sheet. A suite of 17 (or more) indicators are typically considered in an assessment. The ecological site(s) representative of an assessment location must be known prior to applying the protocol and must be verified based on soils and climate. Current plant community cannot be used to identify the ecological site.
Author(s)/participant(s) Contact for lead author Date Approved by Approval date Composition (Indicators 10 and 12) based on Annual Production Indicators
-
Number and extent of rills:
-
Presence of water flow patterns:
-
Number and height of erosional pedestals or terracettes:
-
Bare ground from Ecological Site Description or other studies (rock, litter, lichen, moss, plant canopy are not bare ground):
-
Number of gullies and erosion associated with gullies:
-
Extent of wind scoured, blowouts and/or depositional areas:
-
Amount of litter movement (describe size and distance expected to travel):
-
Soil surface (top few mm) resistance to erosion (stability values are averages - most sites will show a range of values):
-
Soil surface structure and SOM content (include type of structure and A-horizon color and thickness):
-
Effect of community phase composition (relative proportion of different functional groups) and spatial distribution on infiltration and runoff:
-
Presence and thickness of compaction layer (usually none; describe soil profile features which may be mistaken for compaction on this site):
-
Functional/Structural Groups (list in order of descending dominance by above-ground annual-production or live foliar cover using symbols: >>, >, = to indicate much greater than, greater than, and equal to):
Dominant:
Sub-dominant:
Other:
Additional:
-
Amount of plant mortality and decadence (include which functional groups are expected to show mortality or decadence):
-
Average percent litter cover (%) and depth ( in):
-
Expected annual annual-production (this is TOTAL above-ground annual-production, not just forage annual-production):
-
Potential invasive (including noxious) species (native and non-native). List species which BOTH characterize degraded states and have the potential to become a dominant or co-dominant species on the ecological site if their future establishment and growth is not actively controlled by management interventions. Species that become dominant for only one to several years (e.g., short-term response to drought or wildfire) are not invasive plants. Note that unlike other indicators, we are describing what is NOT expected in the reference state for the ecological site:
-
Perennial plant reproductive capability:
Print Options
Sections
Font
AAAAOther
PrintThe Ecosystem Dynamics Interpretive Tool is an information system framework developed by the USDA-ARS Jornada Experimental Range, USDA Natural Resources Conservation Service, and New Mexico State University.
Accessibility statement


